D3.2 Inheritance
Inheritance explains how alleles, chromosomes, meiosis, pedigrees, linkage, variation and statistical tests predict genetic outcomes across generations in inheritance problems.
- Syllabus
- First assessment 2025
- Topic
- D3.2
- Level
- HL
Inheritance explains how alleles, chromosomes, meiosis, pedigrees, linkage, variation and statistical tests predict genetic outcomes across generations in inheritance problems.
diploid parent (two homologous copies of each autosome) → meiosis → haploid gametes (one copy) → fertilization → diploid zygote (two copies again)
| Cell | Chromosome sets | Alleles possible at one autosomal locus |
|---|---|---|
| body cell in a diploid parent | 2n | two alleles, one on each homolog |
| gamete | n | one allele |
| zygote | 2n | one allele from each parent |
Two alleles does not mean two different alleles. A diploid genotype may be homozygous, with matching alleles, or heterozygous, with different alleles.
| Term | Meaning | Example |
|---|---|---|
| gene | DNA sequence with a functional product or role | a gene affecting pea height |
| locus | the gene's position on a chromosome | the height-gene position |
| allele | one sequence version at that locus | T or t |
| genotype | allele combination carried | TT, Tt or tt |
Use genotype for the allele combination, not for the visible trait. A genotype can be written for one locus, several loci or the whole genome, so state the scope when it matters.
A phenotype is an observable or measurable characteristic produced by the genotype, the environment, or an interaction between them.
| Main cause | Example | Why |
|---|---|---|
| genotype | ABO blood group | inherited alleles determine A and B antigens |
| environment | an acquired scar | injury changes tissue without changing inherited alleles |
| genotype × environment | adult height | growth potential interacts with nutrition and health |
The same phenotype can come from different genotypes, and one genotype can produce different phenotypes in different environments. Phenotype alone therefore does not always identify genotype.
Under complete dominance, a dominant allele determines the heterozygous phenotype. A recessive phenotype appears only when no dominant allele is present.
| Genotype | Allele state | Phenotype when T is dominant |
|---|---|---|
| TT | homozygous dominant | tall |
| Tt | heterozygous | tall |
| tt | homozygous recessive | dwarf |
Dominant does not mean better, stronger or more common. It only describes expression in a heterozygote; a harmful or rare allele can be dominant.
Emasculation and isolation prevent self-pollination, so the experimenter knows the parental sources of both gametes. Reciprocal crosses can also test whether switching the pollen and ovule parents changes the result.
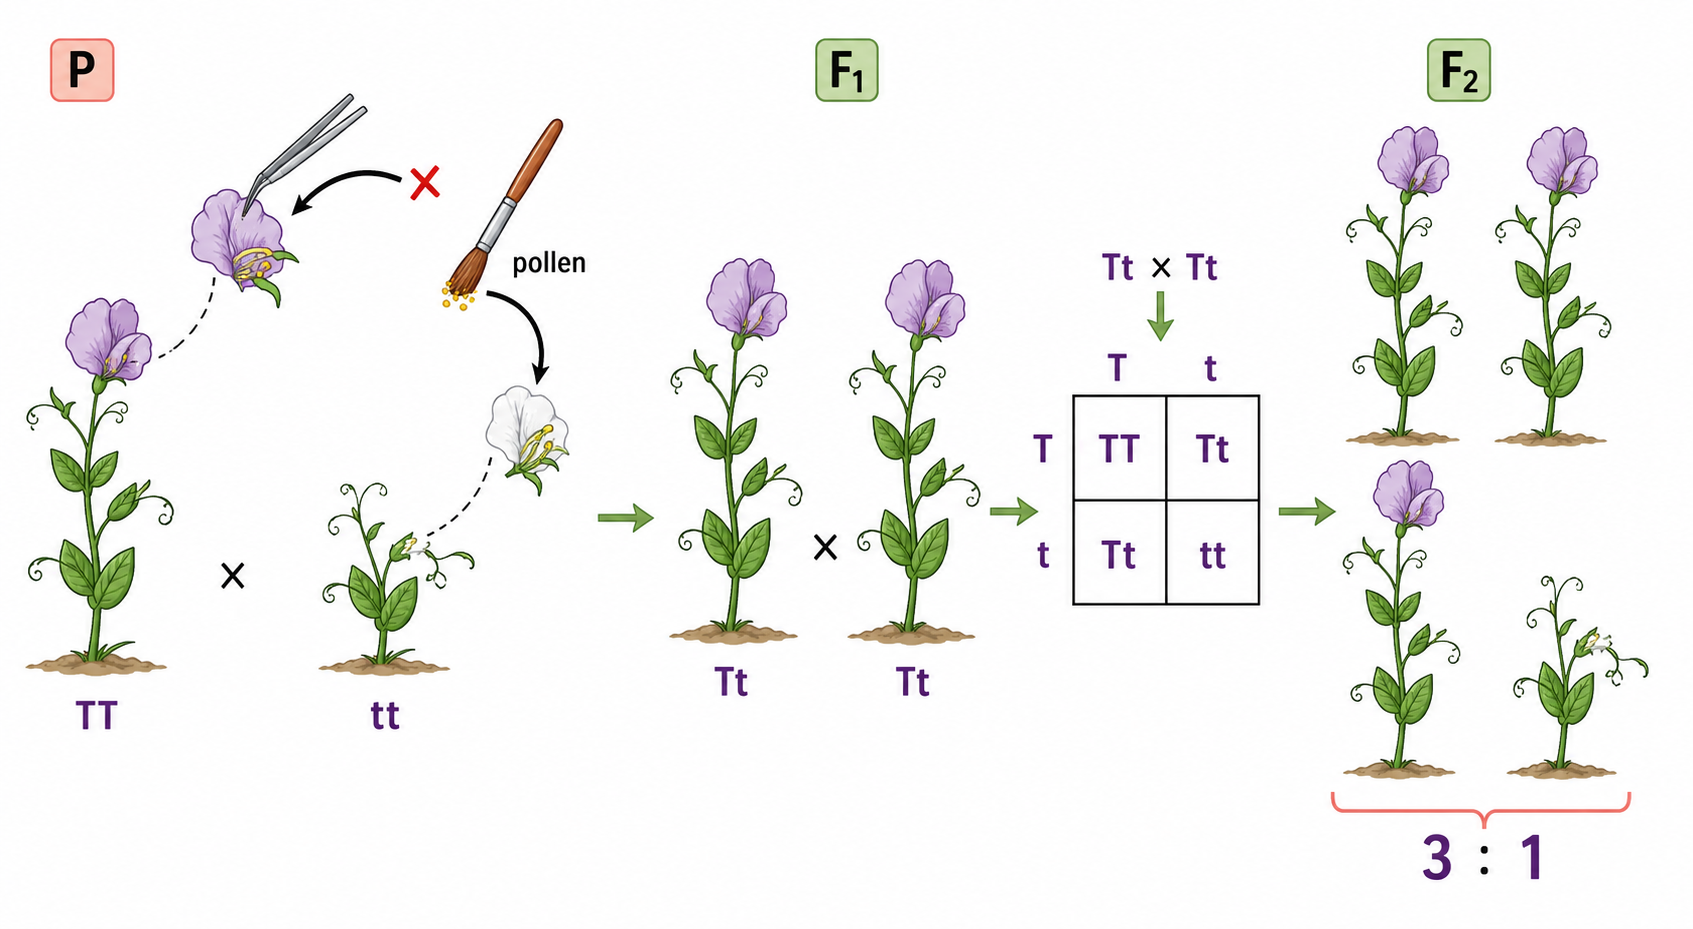
P generation: true-breeding tall TT × true-breeding dwarf tt → every gamete carries T or t, respectively.
F1 generation: every offspring is Tt and tall. The t allele has not blended away; its phenotypic effect is masked in the heterozygote.
F1 self-cross: Tt × Tt → F2 genotypes 1 TT : 2 Tt : 1 tt → phenotypes 3 tall : 1 dwarf in a large sample.
Reappearance of dwarf offspring shows that hereditary factors remain discrete across generations. The observed ratio approaches the probability prediction only when many offspring are counted.
| Tt × Tt | T gamete | t gamete |
|---|---|---|
| T gamete | TT, tall | Tt, tall |
| t gamete | Tt, tall | tt, dwarf |
Each cell has probability 1/4 because each parent produces T and t gametes with probability 1/2. The grid predicts probabilities for each fertilization, not a guarantee that every four offspring will contain one of each cell.
A tall plant could be TT or Tt because both contain the dominant T allele. Cross the unknown plant with a homozygous recessive tester, tt, whose gametes reveal what the unknown parent contributes.
| Unknown parent | Cross with tt | Expected offspring evidence |
|---|---|---|
| TT | TT × tt | all Tt, all tall |
| Tt | Tt × tt | about 1 Tt tall : 1 tt dwarf |
A small all-tall sample does not prove the parent is TT because a heterozygote can produce tall offspring repeatedly by chance. Confidence increases as more offspring are scored.
Phenotypic plasticity is the capacity of one genotype to develop different phenotypes in different environments by changing patterns of gene expression.
environmental cue → signalling pathway → transcription or translation changes → different proteins, cell activity or growth → phenotype better matched to the experienced environment
| Plastic response | Genetic evolution |
|---|---|
| genotype is unchanged within the individual | allele frequencies change across generations |
| can be reversible during a lifetime | inherited population change is not reversed by one individual's environment |
| response range itself can be inherited | selection acts on heritable differences |
A suntan or training response is acquired plasticity; it does not mean the altered phenotype is encoded as a new allele and passed directly to offspring.
two loss-of-function PAH alleles → little or no phenylalanine hydroxylase → phenylalanine is not converted efficiently to tyrosine → phenylalanine and harmful derivatives accumulate → untreated neural development is damaged
| Intervention | Why it helps |
|---|---|
| newborn screening | detects the metabolic problem before severe symptoms appear |
| early low-phenylalanine diet | limits substrate accumulation while still supplying controlled essential phenylalanine |
| continued monitoring | keeps blood concentrations within a safer range as diet and growth change |
The genotype does not change with treatment, but the environment does. Dietary control can greatly change the phenotype, making PKU a clear genotype–environment interaction.
| Genotype | PKU status | Reproductive meaning |
|---|---|---|
| PP | unaffected, not a carrier | passes P |
| Pp | unaffected carrier | can pass P or p |
| pp | affected | passes p |
| Pp × Pp | P gamete | p gamete |
|---|---|---|
| P gamete | PP unaffected | Pp carrier |
| p gamete | Pp carrier | pp affected |
For each pregnancy: 1/4 affected, 1/2 unaffected carrier, 1/4 unaffected non-carrier. The probability resets for every fertilization; previous children do not change the next gamete combination.
Carrier and affected are not synonyms. A heterozygous carrier has a working dominant allele and usually does not show PKU, but can transmit the recessive allele.
A single-nucleotide polymorphism (SNP) is a common difference at one nucleotide position among genomes. A SNP within or near a gene can create or mark a different allele.
| Scale | What may exist at one locus |
|---|---|
| one haploid gamete | one allele |
| one diploid individual | at most two alleles |
| a population gene pool | two, three or many alternative alleles |
Multiple alleles means several versions of one gene in the population. It does not mean that one ordinary diploid person carries every version.
| Phenotype | Possible genotype(s) | Red-cell antigen(s) |
|---|---|---|
| A | IᴬIᴬ or Iᴬi | A |
| B | IᴮIᴮ or Iᴮi | B |
| AB | IᴬIᴮ | A and B |
| O | ii | neither A nor B |
Iᴬ and Iᴮ are codominant because both antigen products appear in IᴬIᴮ. Each is dominant to i, which produces neither A nor B antigen.
Blood group is a phenotype; Iᴬ, Iᴮ and i are alleles. A person with group A or B may hide an i allele, so phenotype does not always identify genotype.
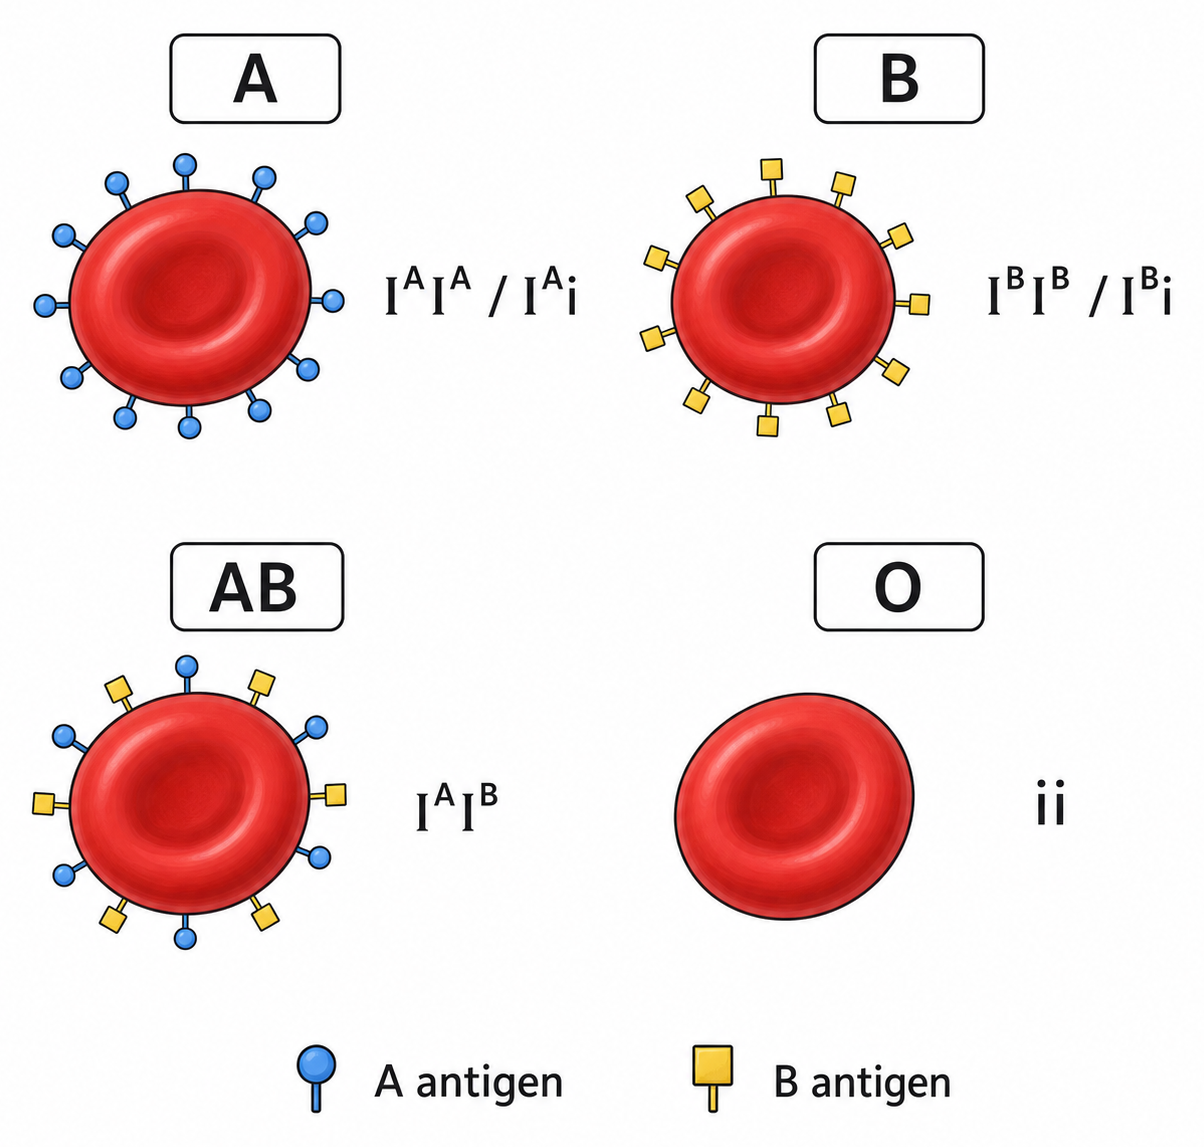
A group-A parent could be IᴬIᴬ or Iᴬi, and a group-B parent could be IᴮIᴮ or Iᴮi. State the genotype assumption before predicting children.
| Iᴬi × Iᴮi | Iᴮ gamete | i gamete |
|---|---|---|
| Iᴬ gamete | IᴬIᴮ, group AB | Iᴬi, group A |
| i gamete | Iᴮi, group B | ii, group O |
With these heterozygous parents, A, B, AB and O phenotypes each have probability 1/4. If either parent is homozygous, the outcome changes.
ABO data can sometimes exclude a proposed parent–child relationship, but common blood groups cannot uniquely prove parentage because many people share the same phenotype and genotype.
| Allele relationship | Heterozygote phenotype | Example |
|---|---|---|
| complete dominance | matches the dominant homozygote | Tt pea is tall |
| codominance | both allele products are detectably expressed | IᴬIᴮ has A and B antigens |
| incomplete dominance | intermediate between the two homozygotes | red × white Mirabilis gives pink F1 |
| Heterozygote × heterozygote | Genotype ratio | Phenotype ratio |
|---|---|---|
| complete dominance | 1:2:1 | 3:1 |
| codominance or incomplete dominance | 1:2:1 | 1:2:1 when all three genotypes are distinguishable |
Codominance is not blending: both products remain identifiable. In incomplete dominance, the heterozygote is intermediate rather than showing two separate products side by side.
P generation: FᴿFᴿ red × FᵂFᵂ white → all FᴿFᵂ pink F1 offspring.
| FᴿFᵂ × FᴿFᵂ | Fᴿ gamete | Fᵂ gamete |
|---|---|---|
| Fᴿ gamete | FᴿFᴿ red | FᴿFᵂ pink |
| Fᵂ gamete | FᴿFᵂ pink | FᵂFᵂ white |
F2 genotype ratio = phenotype ratio = 1 red : 2 pink : 1 white because the heterozygote has its own recognizable phenotype.
Segregation has not changed: each heterozygote still makes the two gamete types equally. The different phenotypic ratio comes from how the heterozygous genotype is expressed.
homologous chromosomes carry two alleles in a diploid parent → meiosis separates one allele into each gamete → fertilization restores a two-allele genotype → allele relationship and environment shape phenotype → offspring data test the prediction
For any genetic cross:
| If the simple 3:1 expectation fails | First question to ask |
|---|---|
| heterozygote has a third phenotype | incomplete dominance? |
| both products appear | codominance? |
| phenotype changes with conditions | environmental or plastic response? |
| more than two alleles occur in the population | multiple-allele locus such as ABO? |
| Gamete contribution | X-bearing sperm | Y-bearing sperm |
|---|---|---|
| X-bearing egg | XX zygote | XY zygote |
| expected probability | about 1/2 | about 1/2 |
Y chromosome with functional SRY → testis-determining factor (TDF) is produced → embryonic gonads develop as testes → testicular hormones direct typical male reproductive development
Without a functional SRY signal, the undifferentiated gonads normally follow ovarian development and typical female reproductive structures develop.
XX/XY is the core human chromosomal model, but chromosome number, SRY location or function, hormone synthesis and tissue response can vary. Chromosomal pattern alone does not describe every aspect of sex or gender.
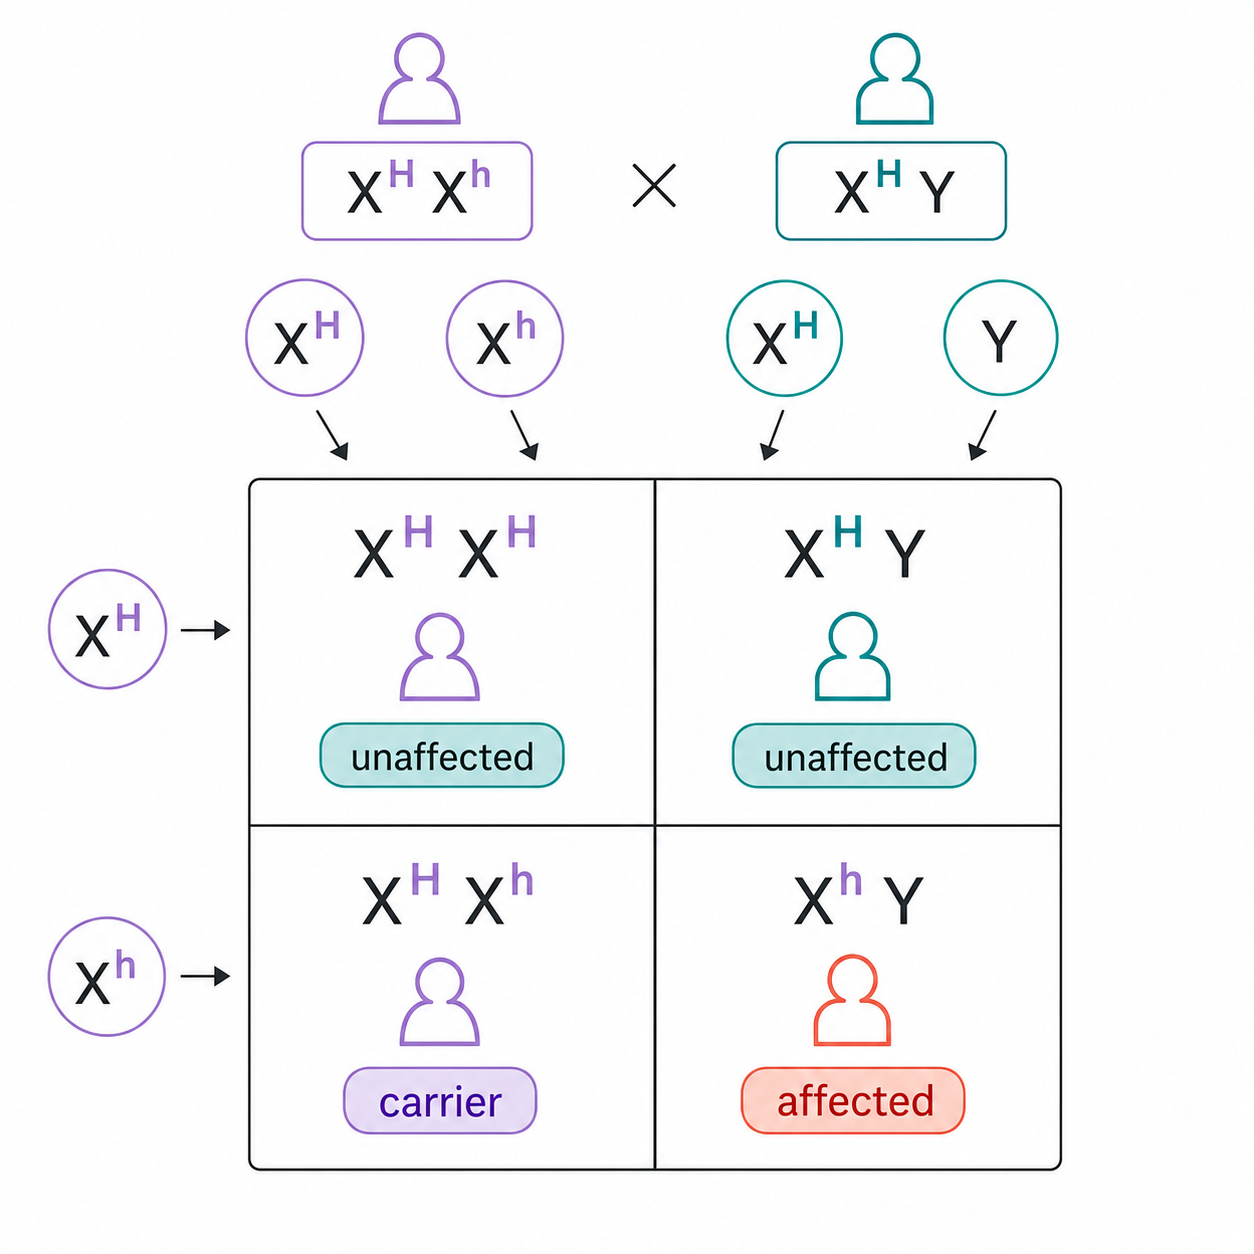
Most genes in the non-homologous region of X have no matching allele on Y. An XY individual is therefore hemizygous for those X-linked genes: the single allele on X is expressed even if it is recessive.
| Genotype | Typical status for an X-linked recessive allele h |
|---|---|
| XᴴXᴴ | unaffected XX |
| XᴴXʰ | unaffected carrier XX |
| XʰXʰ | affected XX |
| XᴴY | unaffected XY |
| XʰY | affected XY |
Write the allele as a superscript on X, such as Xᴴ or Xʰ. Do not place the X-linked allele on Y when the gene is absent from the relevant Y region.
| XᴴXʰ × XᴴY | Xᴴ sperm | Y sperm |
|---|---|---|
| Xᴴ egg | XᴴXᴴ unaffected daughter | XᴴY unaffected son |
| Xʰ egg | XᴴXʰ carrier daughter | XʰY affected son |
Among daughters: 1/2 carriers and 1/2 non-carriers; none affected in this cross. Among sons: 1/2 affected and 1/2 unaffected. Across all offspring, each grid outcome has probability 1/4.
Haemophilia A and B result from deficient clotting factors. The inheritance pattern reflects an X-linked recessive allele; treatment supplies or supports the missing clotting function but does not alter the inherited allele.
| Pedigree mark | Meaning |
|---|---|
| square / circle | male / female in the standard convention |
| filled symbol | individual shows the tracked phenotype |
| horizontal partner line | mating or reproductive partnership |
| vertical descent line | offspring connection |
| shared sibship line | siblings from the same parents |
| I, II, III … | generations |
| 1, 2, 3 … | individuals within a generation |
A pedigree records observed family evidence, not every conception or every relative. Small families and missing records can make more than one inheritance model possible.
| Observation | Strong inference |
|---|---|
| two unaffected parents have an affected child | supports recessive inheritance; contradicts simple complete-dominant inheritance |
| affected person has an affected parent in every generation | supports dominance, but does not prove it alone |
| affected father has an affected son | contradicts X-linked transmission from father to son |
| affected sons arise from unaffected mothers | consistent with X-linked recessive carrier mothers |
| males and females affected similarly | supports autosomal inheritance |
Start with forced genotypes. For an autosomal recessive trait, affected people are aa; each unaffected parent of an affected child must carry a. For an X-linked recessive trait, an affected son XʰY proves that his mother supplied Xʰ.
Treat each inheritance mode as a hypothesis. Predict transmissions that must or cannot occur, compare them with the pedigree, and reject a model only when a relationship contradicts it.
Skipping a generation suggests recessiveness but is not a proof. Chance, incomplete records, late onset and variable expression can obscure the apparent pattern.
| Feature | Continuous variation | Discrete variation |
|---|---|---|
| possible values | many intermediate measurements | separate categories |
| common cause | polygenic effects plus environment | often one or few major loci |
| examples | height, body mass, skin pigmentation | ABO group, biological sex chromosome category |
| useful display | histogram or box plot | bar chart or counts table |
Ask whether the variable is measured on a scale or counted in named categories. Height remains continuous even if a researcher later groups measurements into artificial height bands.
Continuous does not mean every imaginable value must occur in one sample, and discrete does not mean the categories are controlled by only one allele.
In polygenic inheritance, several loci contribute to one characteristic. Different combinations of small allele effects generate many genotypic values rather than a few Mendelian phenotype classes.
many contributing genotypes + nutrition, health, temperature or other environmental effects + genotype-specific responses to those conditions → overlapping phenotypes across a continuous range
| Trait | Genetic contribution | Environmental contribution |
|---|---|---|
| height | many growth-related loci | nutrition, disease and developmental conditions |
| body mass | metabolism and appetite loci | diet, activity and health |
| skin pigmentation | several melanin-related loci | ultraviolet exposure changes melanin production |
Do not confuse multiple genes contributing to one trait with multiple alleles at one gene locus. These are different levels of genetic variation.
A common rule marks values below Q1 − 1.5 × IQR or above Q3 + 1.5 × IQR as outliers. Check the convention used before treating the raw minimum and maximum as whisker ends.
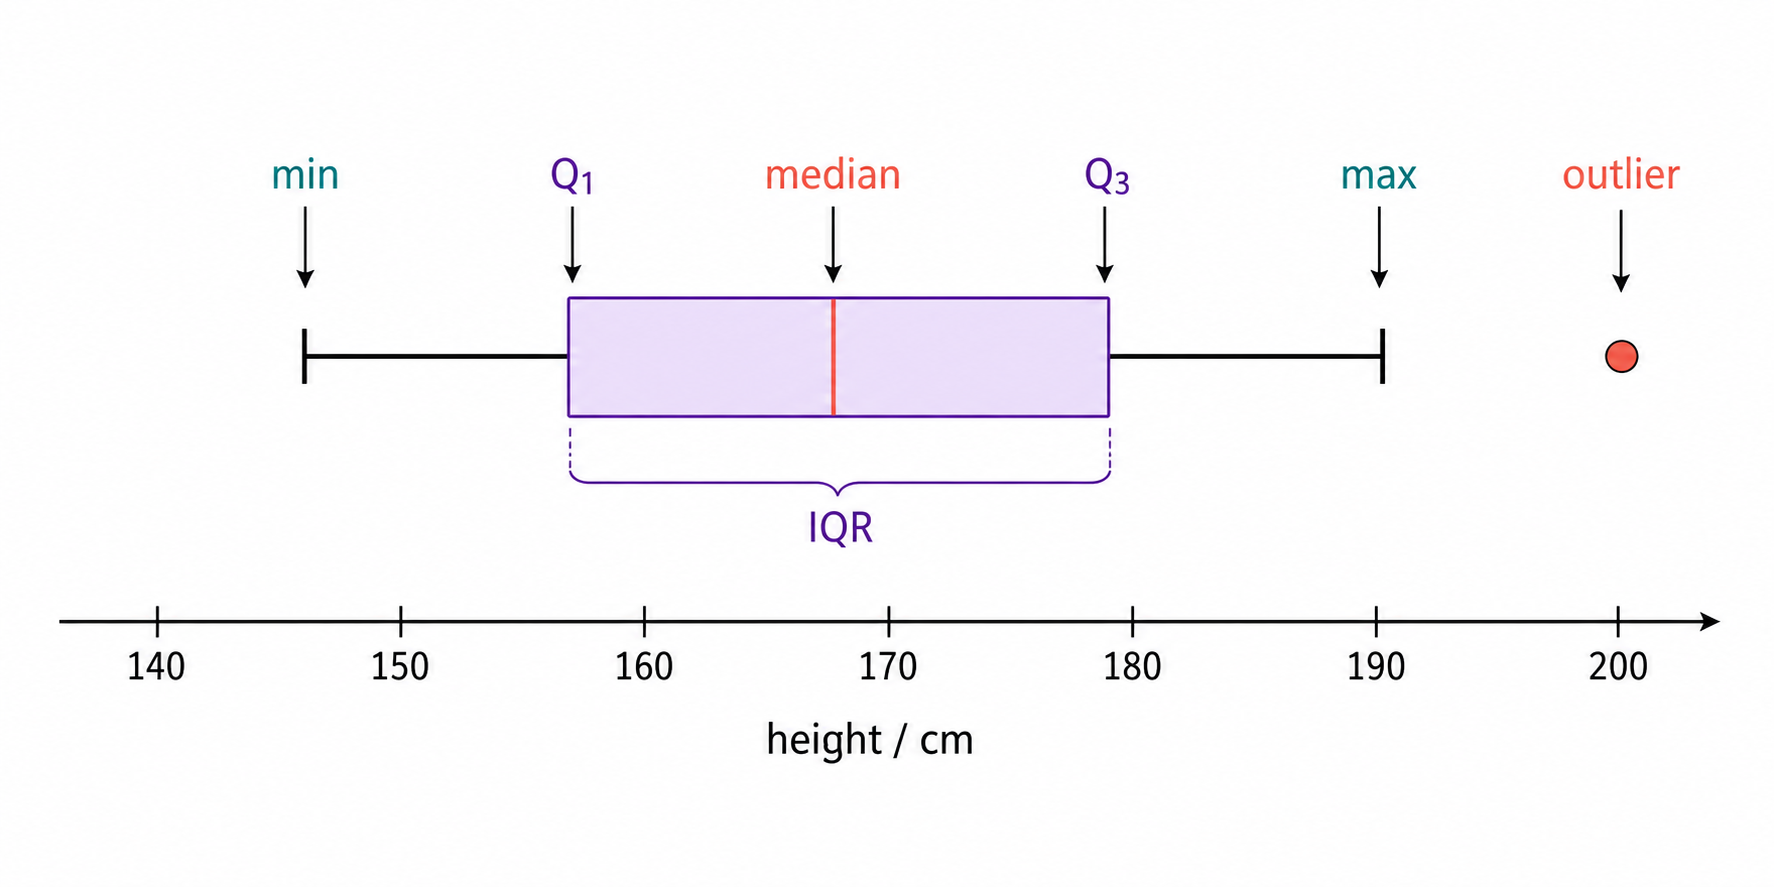
| Feature | What to compare |
|---|---|
| median line | typical central value |
| box length, IQR | spread of the middle 50% |
| whiskers | spread beyond the quartiles among non-outliers |
| isolated points | potential outliers requiring biological or measurement review |
| overlap between boxes | descriptive overlap, not automatically a significance test |
If group A has a higher median but strongly overlapping boxes with group B, report both observations. Do not erase the overlap or claim a significant difference without an appropriate inferential test.
A box plot does not show sample size, separate peaks or every raw value unless these are added. Two very different distribution shapes can share the same median and quartiles.
X and Y contributions establish the usual chromosomal starting point → unequal X-linked gene dosage changes inheritance risk → pedigrees reveal transmission across families → polygenes and environment create continuous population variation → box plots summarize centre and spread
| Evidence source | Reliable question |
|---|---|
| X-linked cross | which parent supplies the allele to sons or daughters? |
| pedigree | which inheritance hypotheses are contradicted by family relationships? |
| continuous measurements | where is the median and how wide is the middle 50%? |
| apparent outlier | biological extreme, data error or different process? |
Match the claim to the evidence scale. One Punnett grid predicts a fertilization probability, a pedigree constrains family genotypes, and a box plot describes a sample distribution; none alone proves a universal biological rule.
Before meiosis, an Aa diploid cell carries A on one homologous chromosome and a at the same locus on the other homolog.
At anaphase I, homologous chromosomes move to opposite poles. A and a therefore enter different daughter cells; meiosis II separates sister chromatids without reuniting the alleles.
If meiotic products survive equally, an Aa parent makes approximately 1/2 A gametes and 1/2 a gametes. Random fertilization then restores two alleles in the zygote.
Mendel's law of segregation is therefore a chromosome-mechanics statement: paired alleles separate because their homologous chromosomes separate during meiosis.
Each bivalent can face either spindle pole at metaphase I. The orientation of the A/a pair does not determine the orientation of a B/b pair on a different chromosome, so maternal and paternal homologs enter daughter cells in different combinations.
| Gene positions | Assortment expectation |
|---|---|
| on different chromosomes | independent |
| far apart on the same chromosome with recombination approaching 50% | behaves approximately independent |
| close together on the same chromosome | linked; parental combinations exceed recombinants |
Independent assortment is not the random separation of sister chromatids. It concerns the relative orientation and separation of different homologous chromosome pairs in meiosis I.
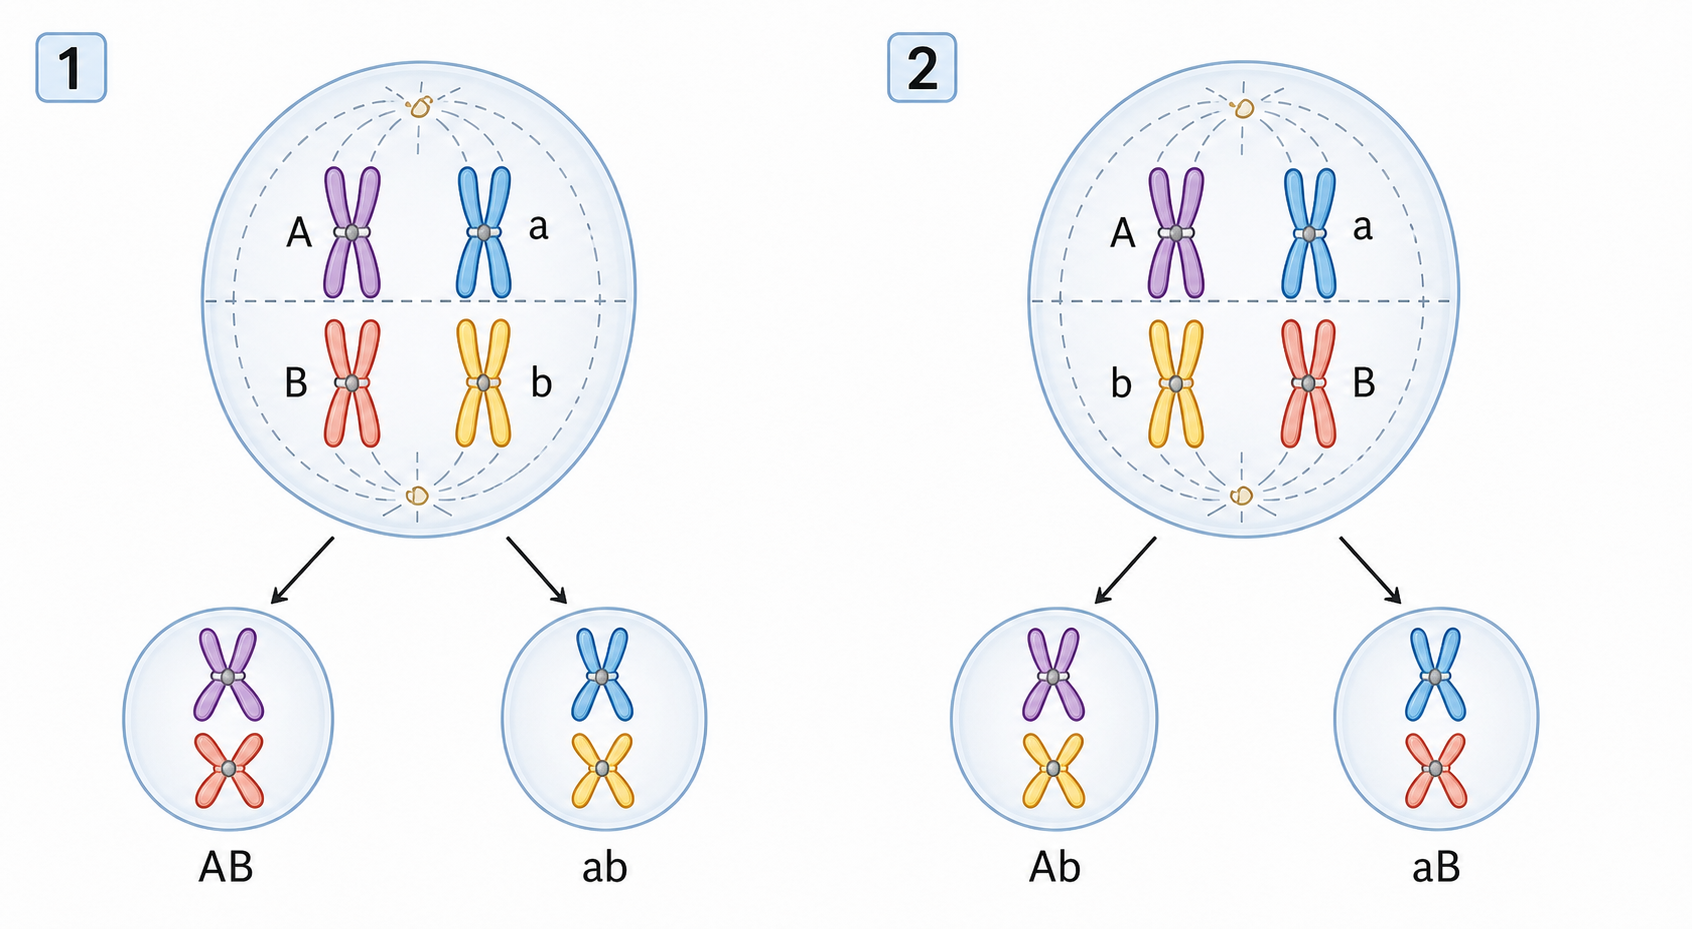
Every gamete from AaBb must contain one allele from the A/a locus and one from the B/b locus. For unlinked loci, multiply the independent probabilities.
| A-locus choice | B-locus choice | Gamete | Probability |
|---|---|---|---|
| A, 1/2 | B, 1/2 | AB | 1/4 |
| A, 1/2 | b, 1/2 | Ab | 1/4 |
| a, 1/2 | B, 1/2 | aB | 1/4 |
| a, 1/2 | b, 1/2 | ab | 1/4 |
A valid gamete list has one allele per locus, no duplicate types and probabilities summing to 1. Writing A, a, B and b as four separate gametes loses one gene from each gamete.
The same multiplication rule scales: an individual heterozygous at n independently assorting loci can make 2ⁿ gamete types, before considering linkage or unequal viability.
Assume both genes are autosomal and unlinked, complete dominance acts at each locus, both parents are AaBb, the four gamete types are equally frequent, fertilization is random and offspring classes survive equally.
| Phenotype class | Probability calculation | Expected fraction |
|---|---|---|
| A_B_ | 3/4 × 3/4 | 9/16 |
| A_bb | 3/4 × 1/4 | 3/16 |
| aaB_ | 1/4 × 3/4 | 3/16 |
| aabb | 1/4 × 1/4 | 1/16 |
The ratio is two independent 3:1 monohybrid probabilities multiplied together. A 4 × 4 grid lists all 16 genotype combinations; the product rule reaches the same phenotype expectation more efficiently.
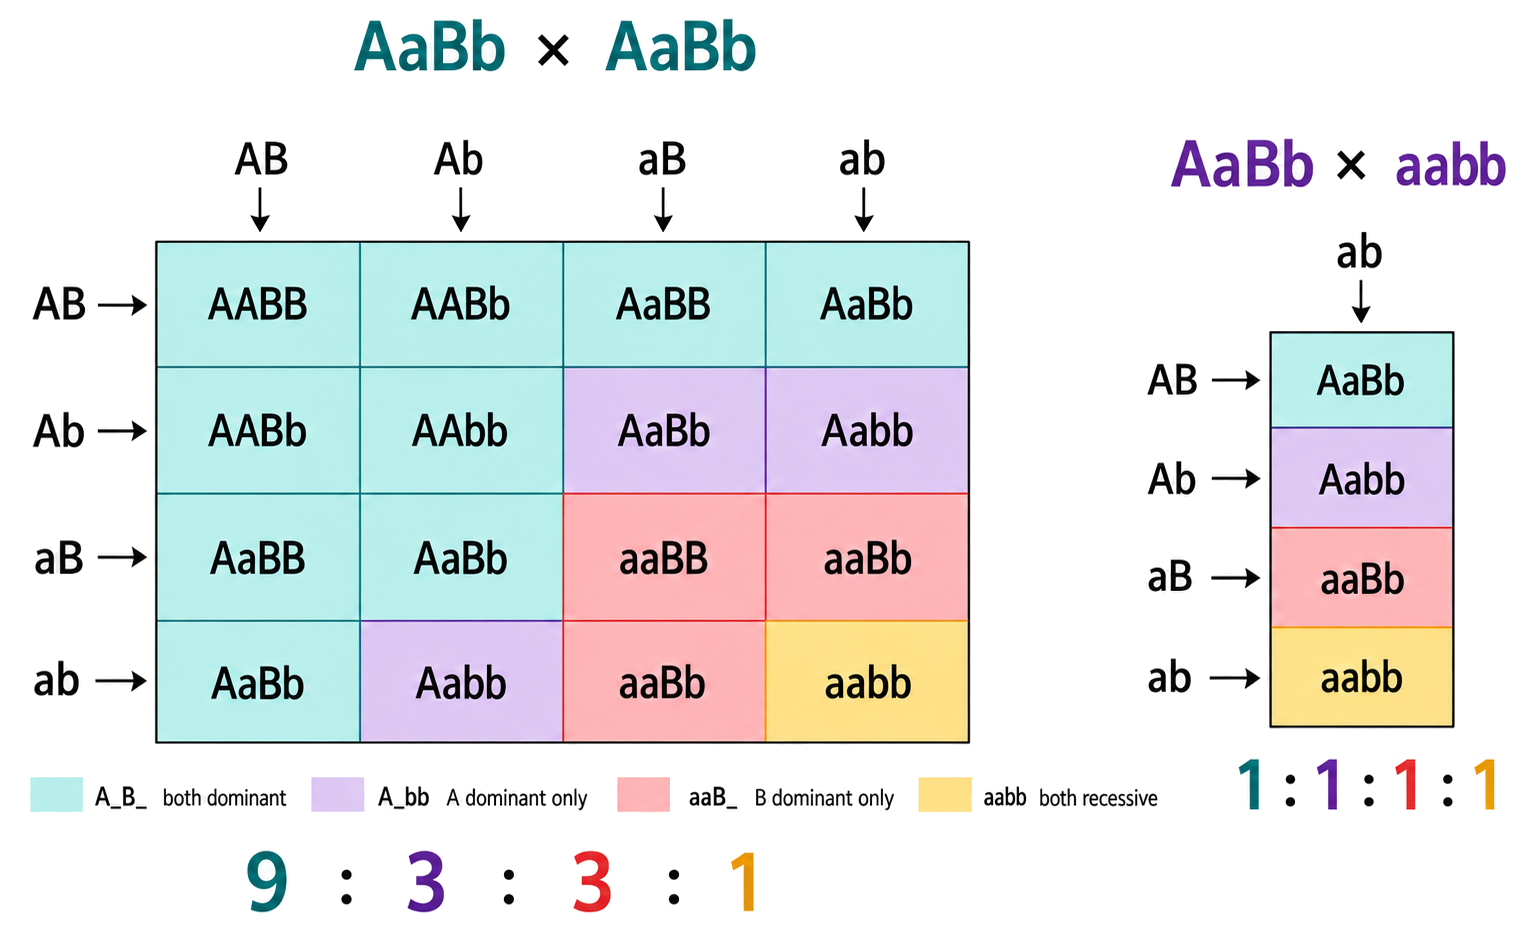
Cross the double heterozygote AaBb with aabb. The tester can contribute only ab, so each offspring genotype reveals which gamete came from the heterozygote.
| AaBb gamete | Tester gamete | Offspring | Phenotype class |
|---|---|---|---|
| AB | ab | AaBb | both dominant |
| Ab | ab | Aabb | A dominant only |
| aB | ab | aaBb | B dominant only |
| ab | ab | aabb | both recessive |
If A/a and B/b assort independently, AB, Ab, aB and ab gametes each occur with probability 1/4, so the test-cross phenotype expectation is 1:1:1:1.
A strong excess of two reciprocal classes and a shortage of the other two suggests linkage: parental chromosome combinations are being transmitted more often than recombinant combinations.
| Database field | Question it answers |
|---|---|
| gene symbol and stable identifier | which gene record? |
| chromosome and genomic coordinates | where is the locus? |
| transcript or product annotation | what is produced? |
| curated functional summary | what evidence supports its role? |
Genes on different chromosomes are unlinked. Genes on the same chromosome are physically linked, but how often crossing over separates them depends on the distance between their loci.
A nearby genomic feature is not automatically the same gene or product. Record the database version, species, coordinates and identifier so the evidence can be checked again.
homologs separate alleles → independently oriented bivalents combine alleles from unlinked genes → AaBb makes AB, Ab, aB and ab gametes equally → random fertilization produces 9:3:3:1 in an F2 or 1:1:1:1 in a test cross
| Prediction | Required conditions |
|---|---|
| 1:1 allele segregation | normal meiosis and equal gamete contribution |
| four equal AaBb gametes | loci unlinked or recombination effectively 50% |
| 9:3:3:1 F2 | complete dominance, random fertilization and equal survival |
| 1:1:1:1 test cross | double heterozygote × double recessive tester |
A database locates the genes; the cross tests their behaviour. If observed offspring depart systematically from the unlinked expectation, inspect chromosome location, parental phase, crossing over and viability before blaming random sampling alone.
| Same AaBb genotype | Alleles on one homolog | Alleles on the other | Name |
|---|---|---|---|
| AB/ab | A with B | a with b | coupling phase |
| Ab/aB | A with b | a with B | repulsion phase |
Writing only AaBb records which alleles are present but loses which combinations share a chromosome. For linked genes, parental phase determines which gametes are common and which require crossing over.
Autosomal linkage means two loci share a non-sex chromosome. Sex linkage is different: it refers to a locus on a sex chromosome, usually X.
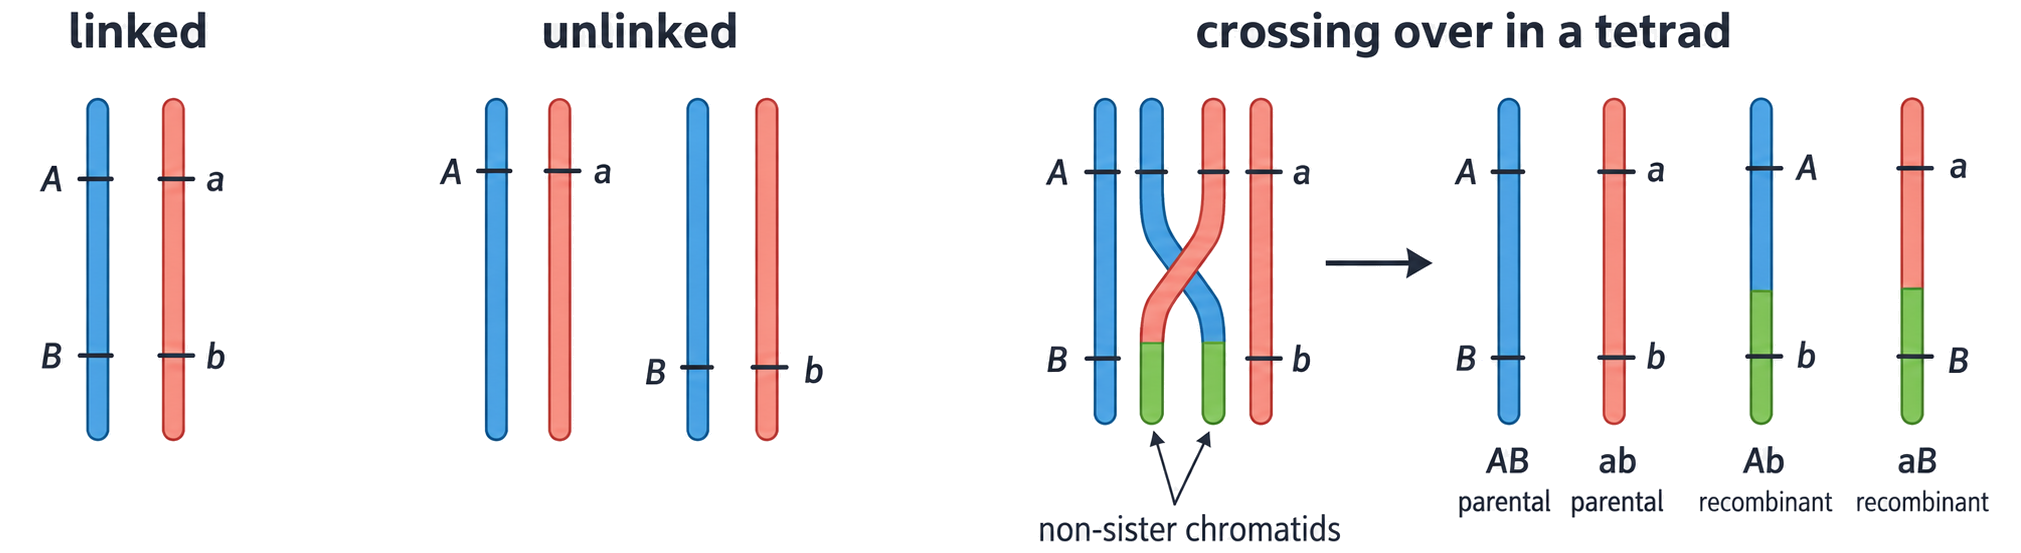
Start with a heterozygote in coupling phase: parental homologs carry AB and ab. After DNA replication, each homolog has two sister chromatids.
A chiasma between the A and B loci exchanges matching segments between non-sister chromatids. Two chromatids remain parental, while two become Ab and aB.
| Chromatid or gamete class | Allele combination | Origin |
|---|---|---|
| parental | AB and ab | no exchange between the loci |
| recombinant | Ab and aB | crossover between the loci |
A crossover elsewhere on the chromosome does not recombine these two loci. The exchange must occur between their positions to separate their parental allele combination.
Cross AB/ab with ab/ab. Because the tester contributes only ab, each offspring's phenotype or genotype identifies the gamete produced by the double heterozygote.
| Heterozygote gamete | Offspring | Classification for AB/ab parent |
|---|---|---|
| AB | AaBb | parental |
| ab | aabb | parental |
| Ab | Aabb | recombinant |
| aB | aaBb | recombinant |
Classify by comparison with the heterozygous parent's chromosome combinations, not by whether an offspring looks common or unusual in the population.
r=NR×100%
Here, R is the number of recombinant offspring and N is the total. If a test cross gives 420 AB, 400 ab, 90 Ab and 90 aB offspring, r = (90 + 90) / 1000 × 100% = 18%.
| Observation | Inference |
|---|---|
| recombinants much below 50% | loci are linked |
| lower recombinant frequency | loci are usually closer, so fewer chiasmata fall between them |
| about 50% recombinants | loci behave as unlinked; they may be on different chromosomes or far apart |
Recombinant frequency does not exceed 50% in an ordinary two-locus test. Multiple crossovers can restore parental combinations, so frequency underestimates large physical distances.
| Statement | Meaning in a dihybrid goodness-of-fit test |
|---|---|
| null hypothesis, H₀ | observed departures from the expected genetic ratio are due to chance sampling |
| alternative hypothesis, H₁ | the departures are too large for that chance model; another explanation is needed |
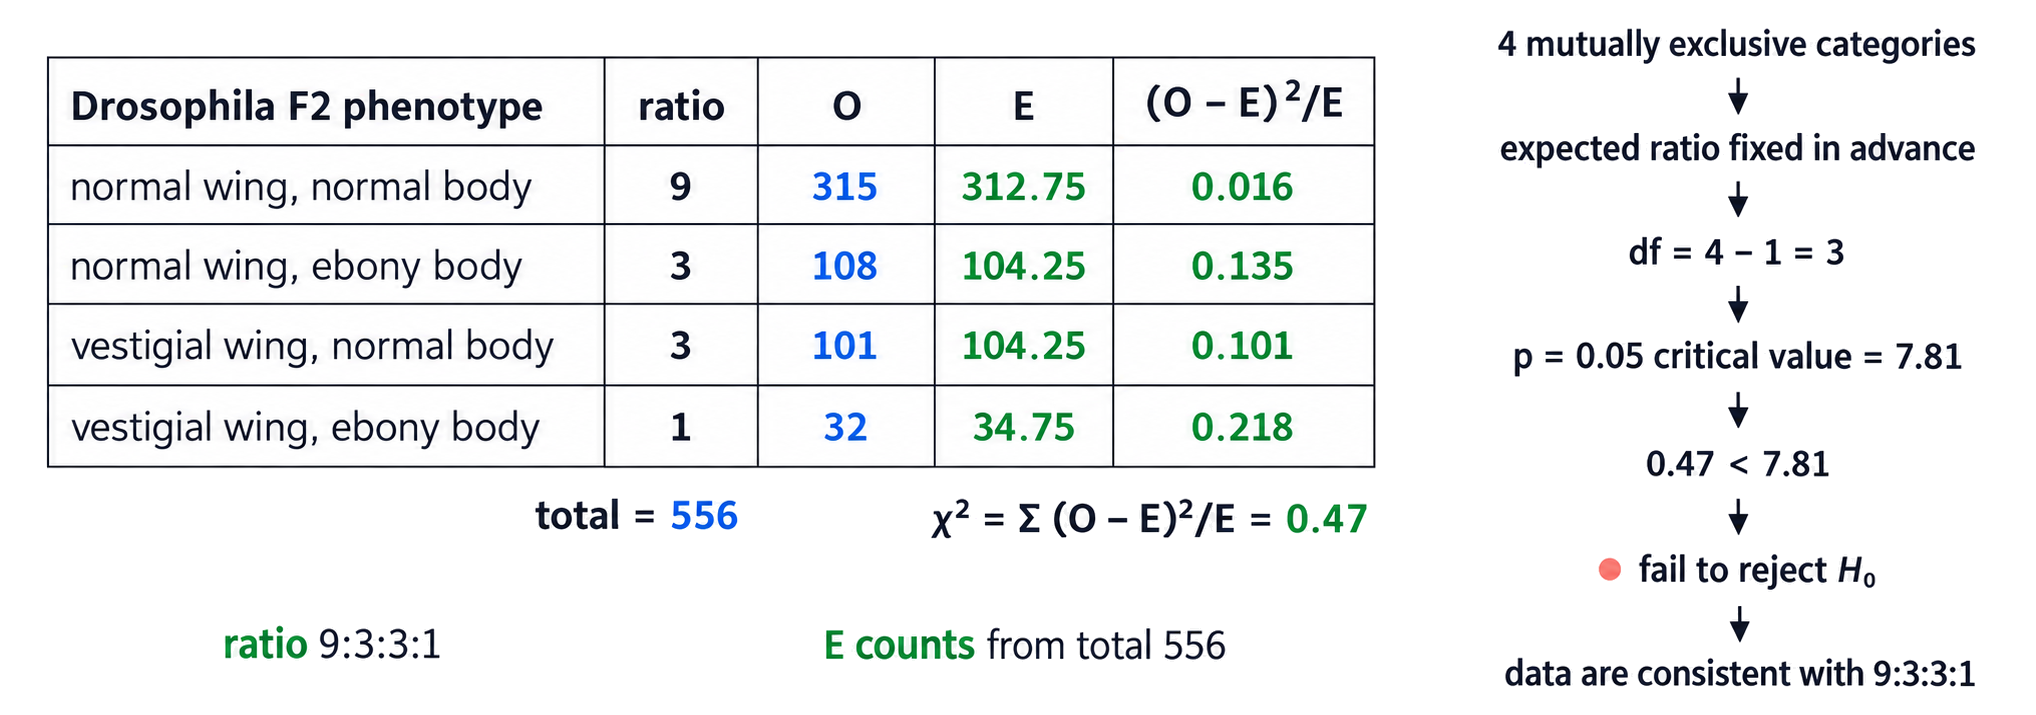
Convert the ratio to expected counts before calculating χ². For a total of 556 offspring and a 9:3:3:1 model: multiply 556 by 9/16, 3/16, 3/16 and 1/16 to obtain 312.75, 104.25, 104.25 and 34.75.
Categories must be mutually exclusive, observations should be independent and expected counts should be large enough for the approximation. The expected ratio must come from a biological model chosen before inspecting the deviations.
Chi-squared tests whether counts fit a specified expectation; it does not identify the true alternative mechanism when they do not fit.
χ2=∑E(O−E)2
| Category | O | E | (O − E)² / E |
|---|---|---|---|
| both dominant | 315 | 312.75 | 0.016 |
| A dominant only | 108 | 104.25 | 0.135 |
| B dominant only | 101 | 104.25 | 0.101 |
| both recessive | 32 | 34.75 | 0.218 |
| sum | 556 | 556 | χ² = 0.470 |
For four mutually exclusive categories with one fixed total and no parameters estimated from the data, degrees of freedom = categories − 1 = 3.
Use counts, not percentages, inside the formula. Keep expected values unrounded during calculation, and include every category contribution before comparing with a critical value.
| At p = 0.05 | Statistical decision | Genetic conclusion |
|---|---|---|
| χ² ≤ critical value | fail to reject H₀ | deviations are not significant; data are consistent with the expected ratio |
| χ² > critical value | reject H₀ | deviations are significant; the stated ratio does not adequately explain the data |
For df = 3, the p = 0.05 critical value is 7.815. Because 0.470 < 7.815, fail to reject H₀: the observed Drosophila counts are consistent with a 9:3:3:1 expectation.
Do not say the test proves H₀ or proves independent assortment. A non-significant result means the observed departure is small enough to be explained by sampling under the model.
A significant result directs further investigation. Possible causes include linkage, differential survival, non-random fertilization, scoring error or an incorrect dominance model; chi-squared alone does not choose among them.
meiosis predicts gamete combinations → chromosome loci determine whether genes assort independently or travel together → crossing over creates reciprocal recombinants → test-cross counts reveal parental phase and recombinant frequency → chi-squared tests whether departures from a chosen ratio exceed chance expectation
| Offspring pattern | First model to examine |
|---|---|
| 9:3:3:1 F2 | two unlinked genes with complete dominance |
| 1:1:1:1 test cross | four equally frequent gametes from an unlinked double heterozygote |
| two large and two small reciprocal test-cross classes | linked loci with crossing over |
| significant χ² departure | assumptions, linkage, viability, fertilization or scoring require review |
Keep prediction and evidence separate: define the genetic model first, calculate expected counts from it, compare observations with the expectation, and change the model only when chromosome location or statistical evidence requires it.
1 mark
For what reason do gametes contain only one allele of each gene?
3 marks
L. purpureus can have purple or white flowers. Two pure-breeding varieties were crossed: HA 4 with white flowers and GL 424 with purple flowers. All of the F1 plants had purple flowers. The F1 plants were self-pollinated to produce an F2 generation. There were 97 plants with purple flowers and 38 plants with white flowers in the F2 generation.
Using a Punnett grid, explain the results of this cross.
1 mark
Define the term genotype.
2 marks
Identify the phenotypes of each part of the phenotypic ratio.
| Ratio | Phenotypes |
|---|---|
| 9 | |
| 3 | |
| 3 | |
| 1 |
4 marks
Many genetic diseases are due to recessive alleles of autosomal genes that code for an enzyme. Using a Punnett grid, explain how parents who do not show signs of such a disease can produce a child with the disease.
1 mark
Scientists incubated larvae of the moth Utetheisa ornatrix at either 15∘C or 22∘C until they hatched. They found the hatched moths had different wing colour patterns due to phenotypic plasticity.
Moth from larvae incubated at \(15^{\circ
Moth from larvae incubated at \(22^{\circ
Which of the following explains the observed differences in wing colour?
4 marks
Discuss the causes and treatments of phenylketonuria.
1 mark
Which statement defines alleles?
9 marks
Describe the inheritance of ABO blood groups.
1 mark
A Mirabilis jalapa plant with red flowers was crossed with one with white flowers. All plants in the F1 generation had pink flowers. What phenotype ratio would be expected in the F2 generation?
4 marks
Distinguish between autosomes and sex chromosomes in humans.
8 marks
Explain how males inherit hemophilia and how females can become carriers for the condition.
2 marks
Explain how the pedigree chart shows that the dominant allele causing PKD is not on the X chromosome.
7 marks
Explain the reasons for variation in human height.
3 marks
Using the data, deduce whether the incidence of CHF or the incidence of anemia has a greater effect on the blood hepcidin concentration.
6 marks
Outline the relationship between Mendel's law of independent assortment and meiosis.
3 marks
The expected ratio of phenotypes in the offspring of a cross between a plant with narrow, yellow leaves and a plant heterozygous for the genes for leaf width and colour is 1: 1: 1: 1.
Justify this expected ratio using a Punnett grid or other diagram.
3 marks
Outline how it can be shown that the genes for shell base colour (Cc) and presence or absence of bands (Bb) are linked.
1 mark
An individual is heterozygous for two linked genes abAB.
To investigate the frequency of crossing over, a test cross is carried out between the individual and another that is homozygous recessive for both genes. What are the possible recombinants in the offspring of this cross?
2 marks
The chi-squared value was calculated as shown. Deduce, with reasons, whether the observed ratio differed significantly from the expected Mendelian ratio.
| Probability | |||||||||||
|---|---|---|---|---|---|---|---|---|---|---|---|
| Degrees of freedom | 0.995 | 0.975 | 0.20 | 0.10 | 0.05 | 0.025 | 0.02 | 0.01 | 0.005 | 0.002 | 0.001 |
| 1 | 0.00004 | 0.001 | 1.642 | 2.706 | 3.841 | 5.024 | 5.412 | 6.635 | 7.879 | 9.550 | 10.828 |
| 2 | 0.010 | 0.051 | 3.219 | 4.605 | 5.991 | 7.378 | 7.824 | 9.210 | 10.597 | 12.429 | 13.816 |
| 3 | 0.072 | 0.216 | 4.642 | 6.251 | 7.815 | 9.348 | 9.837 | 11.345 | 12.838 | 14.796 | 16.266 |
| 4 | 0.207 | 0.484 | 5.989 | 7.779 | 9.488 | 11.143 | 11.668 | 13.277 | 14.860 | 16.924 | 18.467 |
| 5 | 0.412 | 0.831 | 7.289 | 9.236 | 11.070 | 12.833 | 13.388 | 15.086 | 16.750 | 18.907 | 20.515 |
| 6 | 0.676 | 1.237 | 8.558 | 10.645 | 12.592 | 14.449 | 15.033 | 16.812 | 18.548 | 20.791 | 22.458 |
| 7 | 0.989 | 1.690 | 9.803 | 12.017 | 14.067 | 16.013 | 16.622 | 18.475 | 20.278 | 22.601 | 24.322 |