Gene expression connects DNA, transcription regulation, epigenetic control, transcript stability, proteomes and environmental signals to phenotype in living cells and tissues.
Gene Expression Connects DNA Information to Phenotype
HL only
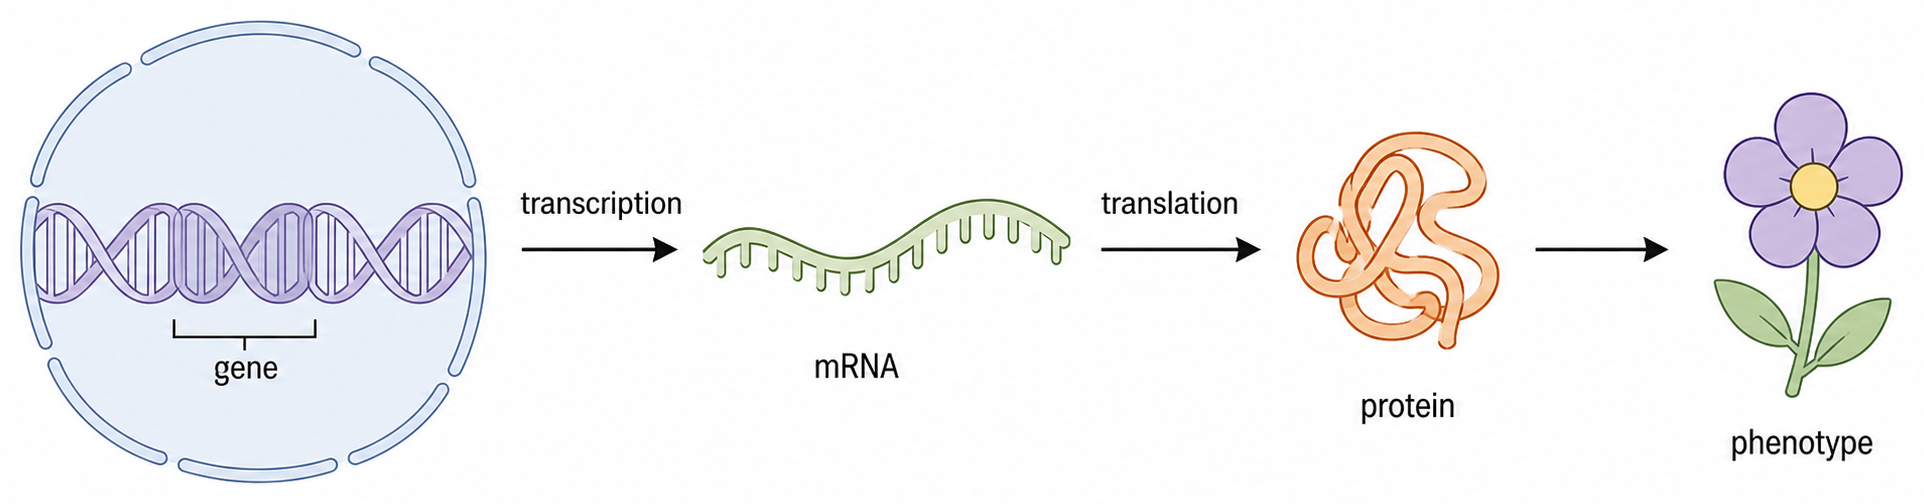
Gene expression is the use of information in a gene to produce a functional RNA or protein whose activity can affect cell structure, cell behaviour and phenotype.
For a protein-coding gene:
DNA base sequence → transcription → mRNA sequence → translation → amino-acid sequence → folded protein and cellular function → contribution to phenotype
A gene does not act on phenotype by itself. Its effect depends on whether it is expressed, how much product is made, what the product does and the cellular or environmental context.
Protein Output Depends on Several Regulated Rates
HL only
The amount of a protein present at one time reflects a balance between its production and removal, not a single on/off switch.
Control point
Immediate effect
Consequence for protein output
transcription initiation
changes how many mRNA molecules are made
changes the number of templates available
mRNA processing and export
changes which mature transcripts reach ribosomes
changes which messages can be translated
mRNA degradation
changes transcript lifetime
changes how many translation rounds can occur
translation rate
changes ribosome use of each mRNA
changes protein production per transcript
protein modification or degradation
changes activity or lifetime of the product
changes functional protein present
More mRNA often permits more translation, but mRNA abundance alone does not determine phenotype: translation efficiency, protein activation and protein lifetime also matter.
The Promoter Organizes Transcription Initiation
HL only
A promoter is a non-coding DNA region near the start of a gene where general transcription factors and RNA polymerase assemble to initiate transcription.
Specific DNA sequences are recognized by proteins → a transcription-initiation complex assembles at the promoter → RNA polymerase is positioned on the template strand → transcription begins at the correct site and direction.
Proteins that stabilize or recruit the initiation complex increase transcription. Proteins that block assembly, polymerase recruitment or promoter access decrease transcription.
The promoter is DNA; a transcription factor is a protein that binds DNA. Neither should be called a gene that codes for the protein being regulated.
Enhancers and Repressors Supply Gene-Specific Inputs
HL only
Sequence-specific transcription factors bind regulatory DNA only when their DNA-binding region matches the target base sequence.
Regulatory input
Binding site
Usual effect
activator
enhancer
helps recruit or stabilize the transcription machinery, increasing transcription
repressor
silencer or other regulatory sequence
interferes with activation, promoter access or initiation, decreasing transcription
An enhancer may lie thousands of base pairs upstream or downstream of its gene. DNA looping can bring enhancer-bound activators into contact with proteins at the promoter.
A gene's transcription rate reflects the combination of regulatory proteins present in that cell. One enhancer does not make a gene permanently active in every tissue.
mRNA Lifetime Sets the Window for Translation
HL only
1
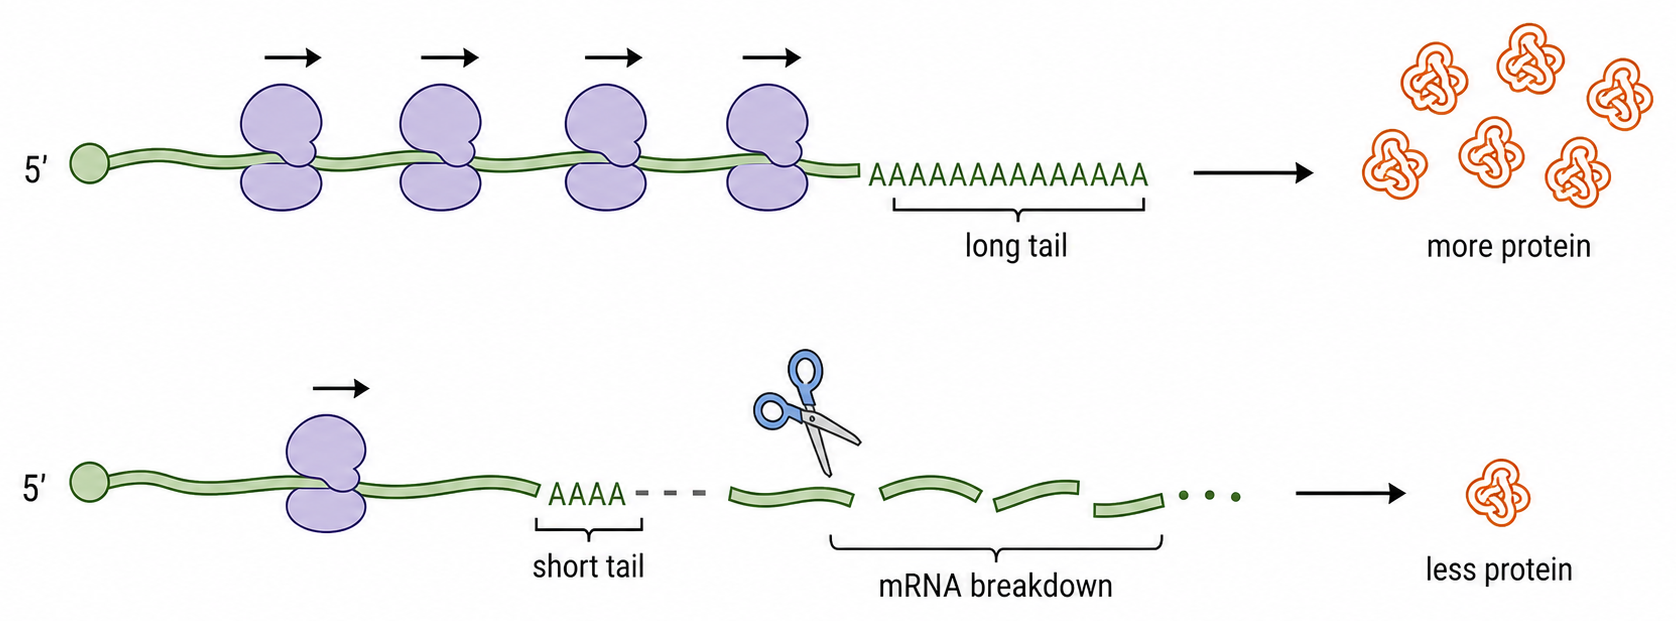
An mRNA can be translated repeatedly while it remains intact and accessible to ribosomes. Regulating its degradation therefore changes how long protein production can continue.
2
poly-A tail shortens → the transcript becomes less stable → protective structures are removed → nucleases degrade the mRNA → fewer further rounds of translation occur
A short mRNA lifetime allows a rapid change in protein production when conditions change. A stable mRNA can sustain output even after new transcription has decreased.
Expression Output Is the Result of a Regulated Flow
HL only
regulatory proteins and chromatin access → transcription initiation → mature mRNA abundance and lifetime → translation → protein activity and lifetime → cellular effect
Observation
First control question to ask
little or no mRNA
is transcription initiation repressed or is mRNA rapidly degraded?
abundant mRNA but little protein
is translation inefficient or is protein rapidly removed?
protein present but no expected effect
is the protein inactive, misplaced or missing a required partner?
Gene expression is not simply gene present versus gene absent. Explain a change by naming the regulated stage and tracing its consequence to functional protein and phenotype.
Epigenesis Builds Specialized Cell Types from One Zygote
HL only
Epigenesis is the development of organized patterns of cell differentiation from an initially undifferentiated zygote.
one zygote → repeated mitosis → cells receive different positional or signalling inputs → different genes remain active or inactive → different proteins accumulate → cells acquire specialized structures and functions
A pancreatic β cell expresses proteins for insulin production and secretion.
A skeletal-muscle fibre expresses abundant contractile proteins.
A neuron expresses receptors, ion channels and synaptic proteins suited to signalling.
Differentiation usually changes which genes are expressed, not which genes the cell possesses. Most somatic cell types retain essentially the same genome.
Genome, Transcriptome and Proteome Describe Different Layers
HL only
Layer
What it contains
How it changes
genome
the complete DNA information of a cell
relatively stable across most somatic cells
transcriptome
all RNA transcripts present in a cell or tissue at a stated time
changes with cell type, signals and developmental stage
proteome
all proteins present in a cell, tissue or organism at a stated time
changes through translation, modification, location and degradation
The genome supplies possible information. The transcriptome records which regions are being expressed as RNA now. The proteome records the protein products actually present after further regulation.
The transcriptome and proteome must be tied to a sample and time. Neither is a permanent list of everything the genome could produce.
A Shared Genome Can Produce Distinct Cell Identities
HL only
Cells produced from the same zygote usually share the same genome, but regulatory states make different subsets of that genome accessible and active.
Same underlying genome
Different active output
Functional consequence
insulin gene present
abundant insulin mRNA and protein in pancreatic β cells
blood-glucose regulation
collagen genes present
high collagen expression in many connective-tissue cells
extracellular support
ion-channel genes present
neuron-specific channel and receptor profile
electrical signalling
regulatory state → selected transcriptome → selected proteome → specialized structure and function
A cell type does not normally lose every gene it does not use. Inactivity and absence are different claims.
Promoter DNA Methylation Usually Reduces Transcription
HL only
DNA methylation adds methyl groups to particular cytosines without changing the DNA base sequence. Dense methylation in a promoter is usually associated with reduced transcription of the downstream gene.
promoter cytosines become methylated → proteins that recognize methylated DNA can bind and recruit chromatin-compacting machinery → transcription factors and RNA polymerase gain less access → transcription decreases
Because methyl groups can be added, maintained or removed by enzymes, promoter methylation is potentially reversible even when the underlying gene sequence is unchanged.
The regulatory effect of methylation depends on its location. A methyl group anywhere in a gene does not automatically switch that gene off.
Histone Tags Change Chromatin Access in Different Ways
HL only
DNA wraps around histone proteins in nucleosomes. Chemical modification of histone tails changes which proteins associate with chromatin and how accessible nearby DNA is to transcription machinery.
Histone modification
Typical interpretation
Important condition
acetylation
often loosens chromatin and supports transcription
the effect reflects recruitment of acetyl-binding and chromatin-remodelling proteins
deacetylation
often supports compact, less accessible chromatin
reduced access can lower transcription
methylation
may activate or repress transcription
the effect depends on the amino acid and methylation state
Promoter DNA methylation is usually taught as repressive, but histone methylation is not automatically repressive. Its meaning depends on the modified histone site.
Epigenetic inheritance transmits a gene-expression state without transmitting a new DNA base sequence.
During DNA replication, each daughter DNA molecule initially contains one parental strand carrying the previous local methylation pattern and one newly synthesized strand.
2
Maintenance enzymes recognize those local cues and restore methylation or chromatin features on the new material, so daughter cells inherit a similar regulatory state.
This cellular memory helps a dividing liver cell lineage remain different from a dividing skin or muscle cell lineage even though their genomes are very similar.
Persistence through mitosis is not the same as transmission to offspring. Gamete development and early embryos erase many epigenetic marks.
Environmental Signals Can Redirect Gene Expression
HL only
An external factor changes gene expression only through a biological sensing and regulatory pathway: signal or exposure → receptor, metabolic sensor or cellular damage response → regulatory proteins or chromatin change → altered transcription or translation.
Examples include:
light cycle altering transcription in photosynthetic organisms or seasonal tissues
diet, drugs, temperature or pollutants altering signalling and sometimes epigenetic tags
The molecular change may alter a cell's proteome; coordinated changes across many cells can alter physiology or phenotype.
The environment does not rewrite genes because an organism needs a trait. It changes regulatory inputs, and some exposures may also damage DNA through separate mutagenic mechanisms.
Air-Pollution Studies Link Exposure, Epigenetic Change and Lung Disease
HL only
Traffic-related pollution includes particulate matter, ozone, carbon monoxide and nitrogen oxides. Exposure has been associated with altered DNA or histone methylation patterns and with respiratory inflammation or disease.
pollutant exposure → oxidative stress or inflammatory signalling in lung tissue → altered regulatory or epigenetic state → changed expression of inflammatory and repair genes → possible contribution to chronic tissue damage
Evidence
What it supports
What it does not prove alone
exposure correlates with methylation difference
pollution may influence regulation
that methylation caused the disease
methylation correlates with altered expression
the tag may mark a regulatory change
that no other pathway contributed
disease risk rises with exposure
exposure is a risk factor
that every exposed individual will develop disease
A strong conclusion separates observation from mechanism: pollution-related epigenetic change is a plausible contributor, not automatically the only cause of a lung condition.
Epigenetic Reprogramming Resets Most Gamete-Acquired States
HL only
During germ-cell development and early embryonic development, extensive epigenetic reprogramming removes most existing tags so the new organism can establish appropriate developmental expression patterns.
Most environmentally acquired or tissue-specific states are not transmitted unchanged.
Early embryonic genes can be activated rather than remaining locked in a parental tissue pattern.
A small set of parent-of-origin imprints escapes complete resetting or is re-established during gamete formation.
Evidence that an epigenetic mark persists in a person's somatic cells does not by itself show that the mark will pass through gametes to descendants.
Genomic Imprinting Makes Expression Depend on Parent of Origin
HL only
In genomic imprinting, an epigenetic mark causes one parental allele to be expressed differently from the other. The active copy depends on whether the allele came from the mother or father.
Inheritance at an imprinted locus
Expression after fertilization
maternal allele carries the silencing imprint
paternal allele is the working copy
paternal allele carries the silencing imprint
maternal allele is the working copy
Because only one allele may be active, deletion, mutation or abnormal imprinting of that active parental copy can have a phenotype even when the other DNA copy is present but epigenetically silent.
Imprinting does not mean the maternal and paternal alleles have different base sequences. It describes parent-specific regulation of expression.
Epigenetic Regulation Balances Memory with Resetting
HL only
shared genome → cell-specific regulatory and epigenetic state → cell-specific transcriptome → cell-specific proteome → differentiated structure and function
Process
What remains continuous?
What can change?
mitosis in a differentiated lineage
much of the expression state
reversible tags and regulatory inputs
environmental response
DNA base sequence usually remains
signalling, transcription and sometimes epigenetic marks
gamete and early-embryo reprogramming
genome and selected imprints
most parental epigenetic patterns are reset
For any epigenetic claim, ask where the tag is, how it changes access or protein binding, whether it persists through mitosis or gametes, and whether the evidence shows correlation or causation.
Twin Comparisons Separate Shared Genes from Different Environments
HL only
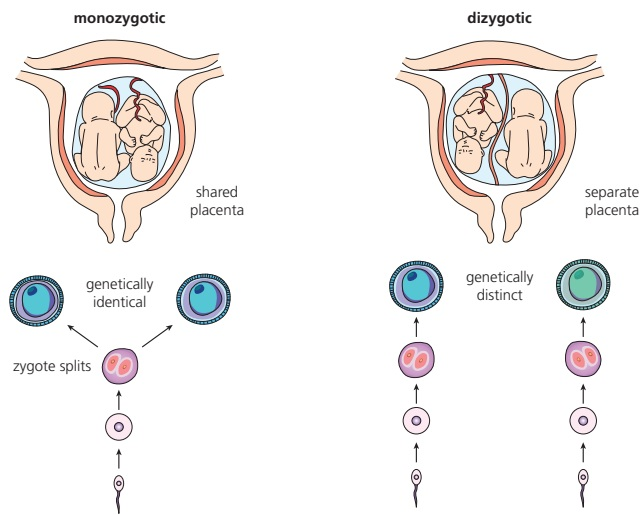
Monozygotic twins develop when one zygote splits and therefore begin with nearly identical genomes. Dizygotic twins develop from two separate fertilizations and share, on average, about half of their segregating genetic variation.
Comparison
Main use
monozygotic twins reared together
holds genome similar while observing outcomes within a largely shared environment
monozygotic twins reared apart
holds genome similar while increasing environmental differences
monozygotic versus dizygotic twin similarity
asks whether greater genetic similarity is associated with greater trait similarity
Monozygotic twins are not biologically identical in every respect. Developmental chance, somatic mutations, epigenetic divergence and non-shared experiences can produce differences.
Twin Similarity Supports Contributions, Not Single-Cause Proof
HL only
Pattern in a sufficiently large study
Supported inference
monozygotic pairs are more similar than dizygotic pairs
genetic differences probably contribute to variation
twins reared together are more similar than comparable twins reared apart
shared environment probably contributes
older or differently exposed monozygotic twins show epigenetic divergence
lifetime environment or stochastic development may alter regulation
Check sample size, how the trait was measured, whether environments were truly different, whether twins were selected representatively, and whether age, sex or socioeconomic conditions confound the comparison.
A trait can reflect gene–environment interaction. High similarity does not mean genes act independently of environment, and a difference within a monozygotic pair does not identify one environmental cause by itself.
Steroid Hormones Turn an External Signal into Transcriptional Control
HL only
1
A lipid-soluble steroid hormone can cross the plasma membrane and bind an intracellular receptor. Ligand binding changes the receptor into an active transcription-regulating complex.
The hormone enters a target cell and binds its specific receptor. The receptor changes conformation, may dimerize and becomes able to regulate transcription.
2
The activated complex enters or acts in the nucleus, binds a hormone-response DNA sequence and recruits coactivators or corepressors, changing target-gene transcription.
Only cells with the required receptor and accessible target regulatory sequences respond directly. The same hormone can therefore cause different expression changes in different tissues.
The hormone is the signal, not the transcription factor's DNA target. The activated receptor complex regulates transcription by binding specific DNA sequences with other regulatory proteins.
An Operon Coordinates Several Bacterial Genes as One Unit
HL only
An operon is a group of adjacent bacterial structural genes controlled together and transcribed from one promoter into a shared mRNA.
Component
Function
regulator gene
encodes a regulatory protein such as a repressor; it may lie outside the operon
promoter
RNA polymerase binding and transcription-start region
operator
DNA site where a regulatory protein can block or permit transcription
structural genes
encode related proteins, often enzymes in one pathway
terminator
signals the end of transcription
Coordinated transcription allows a bacterium to make a complete pathway when it is useful and avoid spending energy and materials on several unnecessary enzymes.
The operator is a DNA binding site, not a protein. The repressor is the protein that binds it. Operons are characteristic of prokaryotic gene organization, not the usual organization of eukaryotic genes.
Lactose Induces the lac Operon by Releasing Repression
HL only
1
Without lactose, the lac repressor has a shape that binds the operator. This obstructs productive RNA-polymerase transcription of the lactose-use structural genes, so the operon is off or expressed only at very low basal levels.
2
When lactose is available, its inducer form binds the repressor allosterically → repressor shape changes → the operator is released → RNA polymerase transcribes the structural genes → enzymes for lactose uptake and metabolism are produced.
The lac operon is inducible: its default repressed state is relieved by substrate availability. When the inducer is depleted, the repressor can bind the operator again.
Tryptophan Represses the trp Operon by Activating Its Repressor
HL only
1
When tryptophan is scarce, the trp repressor is inactive and has little affinity for the operator. RNA polymerase transcribes the structural genes, producing enzymes that synthesize tryptophan.
2
When tryptophan accumulates, it binds the repressor as a corepressor → repressor conformation changes → the active complex binds the operator → transcription of tryptophan-synthesis genes is inhibited.
This is negative feedback: the pathway's product helps switch off further production of the enzymes that make it.
The trp operon is repressible: it is normally available for transcription but can be switched off by abundant product. Tryptophan does not induce the operon.
lac and trp Operons Reverse the Effector Logic
HL only
Dimension
lac operon
trp operon
pathway role
lactose uptake and breakdown
tryptophan synthesis
default regulatory state
repressor active; operon off
repressor inactive; operon available
small effector
lactose-derived inducer
tryptophan corepressor
effector action
inactivates repressor
activates repressor
useful outcome
enzymes made when substrate is present
enzymes withheld when product is abundant
To predict the state, ask two questions: does the small molecule activate or inactivate the repressor, and does the resulting repressor bind the operator?
Both systems conserve resources, but they do so with opposite default states. Do not memorize only that a nutrient is present; trace its effect on repressor shape and operator occupancy.
Signals Change Expression by Altering Regulatory Protein Activity
HL only
external molecule → binds a receptor or regulatory protein → protein conformation, location or DNA binding changes → transcription changes → mRNA and protein abundance change → cell response
selected eukaryotic genes increase or decrease transcription
lac operon
repressor binds lactose-derived inducer
repressor leaves operator
lactose-use genes are transcribed
trp operon
repressor binds tryptophan corepressor
active repressor occupies operator
tryptophan-synthesis genes are repressed
Gene regulation is specific because the responding cell must contain the matching receptor or regulator and the target DNA sequence. The same external condition therefore does not activate every gene or every cell.
Gene expression mechanism
HL only
1 mark
One important chemical in the mobilization of stem cells is a protein, CXCL12, which maintains the stem cells inside the bone marrow. The breakdown of CXCL12 causes the mobilization of stem cells to the blood vessels.
The graph below shows the mobilization of stem cells and the production of mRNA for CXCL12 when the bone marrow is treated with two different chemicals (isoprenaline and clenbuterol).
Explain how the amount of mRNA for CXCL12 gives an indication of the amount of protein CXCL12 produced.
Regulation of transcription
HL only
7 marks
Explain how gene expression can be regulated during transcription to determine an organism's phenotype.
Genome, transcriptome, proteome
HL only
1 mark
Which statement correctly describes genome and proteome?
Epigenetic tags
HL only
2 marks
Explain how methylation of nucleosomes affects DNA transcription.
Environmental effects on expression
HL only
3 marks
Using the data in the bar chart, discuss the evidence for Arabidopsis plants adapting to different daylight regimes by changing the pattern of gene expression.
Epigenetic tag removal
HL only
3 marks
Very soon after fertilization, parental epigenetic methylation is reversed in the DNA. Later, tissue-specific epigenetic modifications are made to the embryonic DNA. The graph follows the degree of methylation from different sources during embryonic development.
According to the graph, what are the changes in DNA methylation during embryonic development?
Monozygotic twin studies
HL only
3 marks
Analyse the data to find whether it supports the hypothesis that genetic factors cause some people to have a much higher chance of cocaine dependence than others.