A virus is a particle that borrows a cell's machinery
HL only
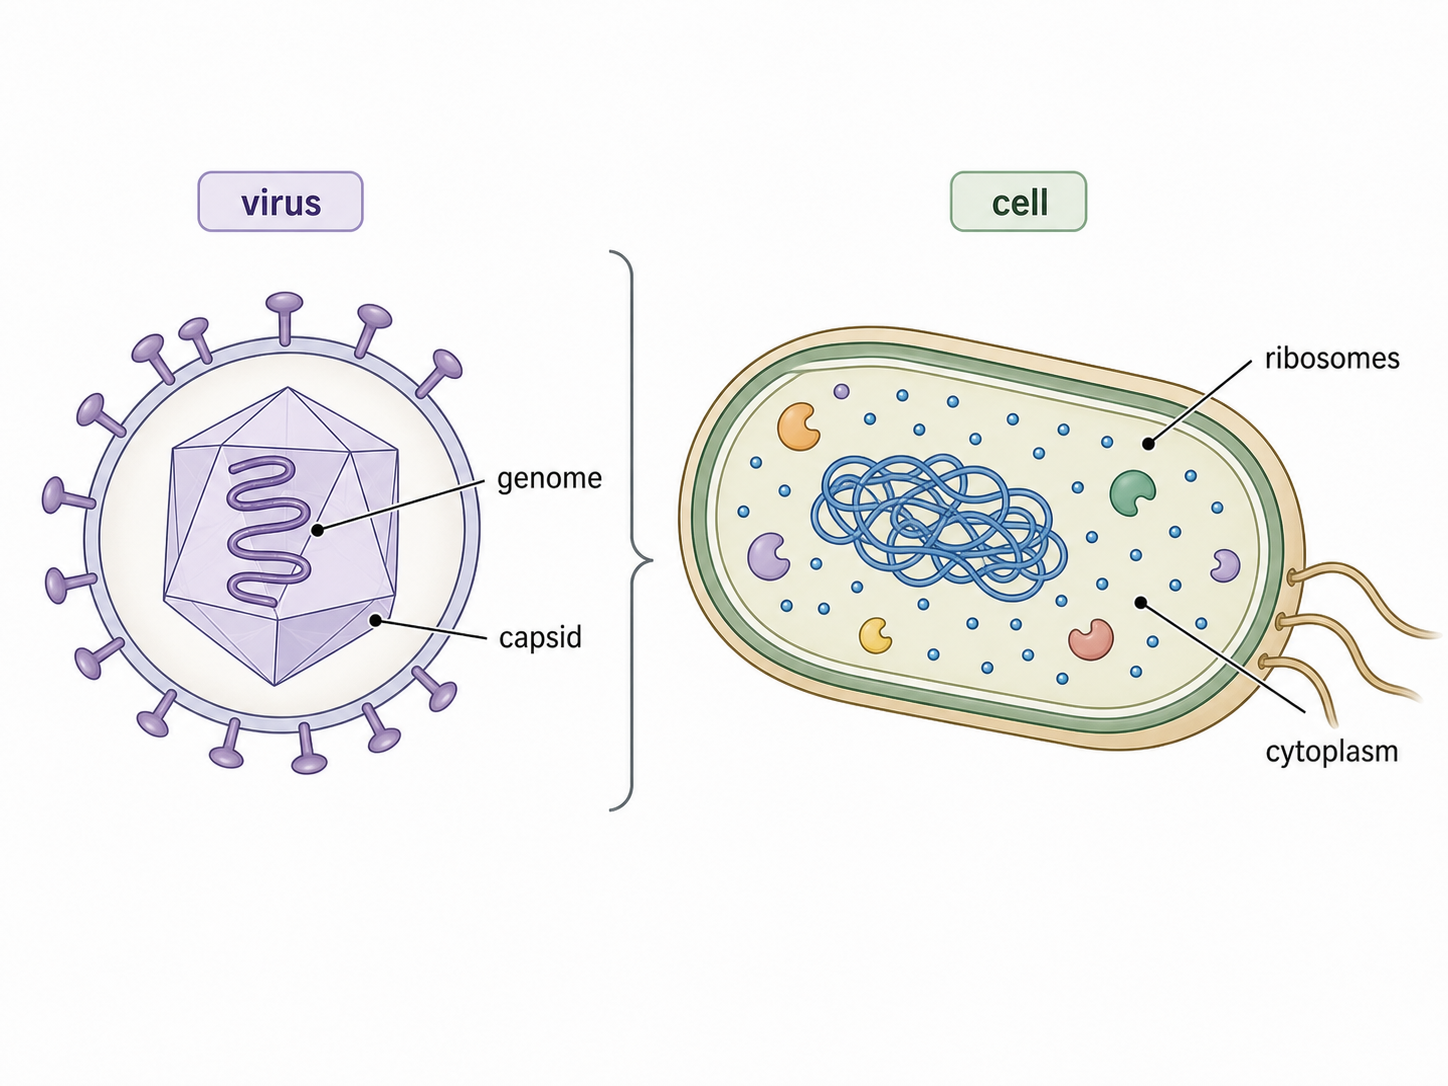
A virion is an infectious, non-cellular particle outside a host cell. Every virus contains a DNA or RNA genome protected by a protein capsid, but it is not a small cell.
Viruses lack the systems needed for independent life:
no cytoplasm in which to maintain metabolism
no ribosomes for protein synthesis
few or no metabolic enzymes
no independent supply of energy or raw materials
A virus is therefore an obligate intracellular parasite: its genome can be copied and expressed only after it enters a compatible host and redirects the host's enzymes, ribosomes, energy and materials. Outside a host, the virion does not grow, metabolize or reproduce.
Virus structure varies along independent axes
HL only
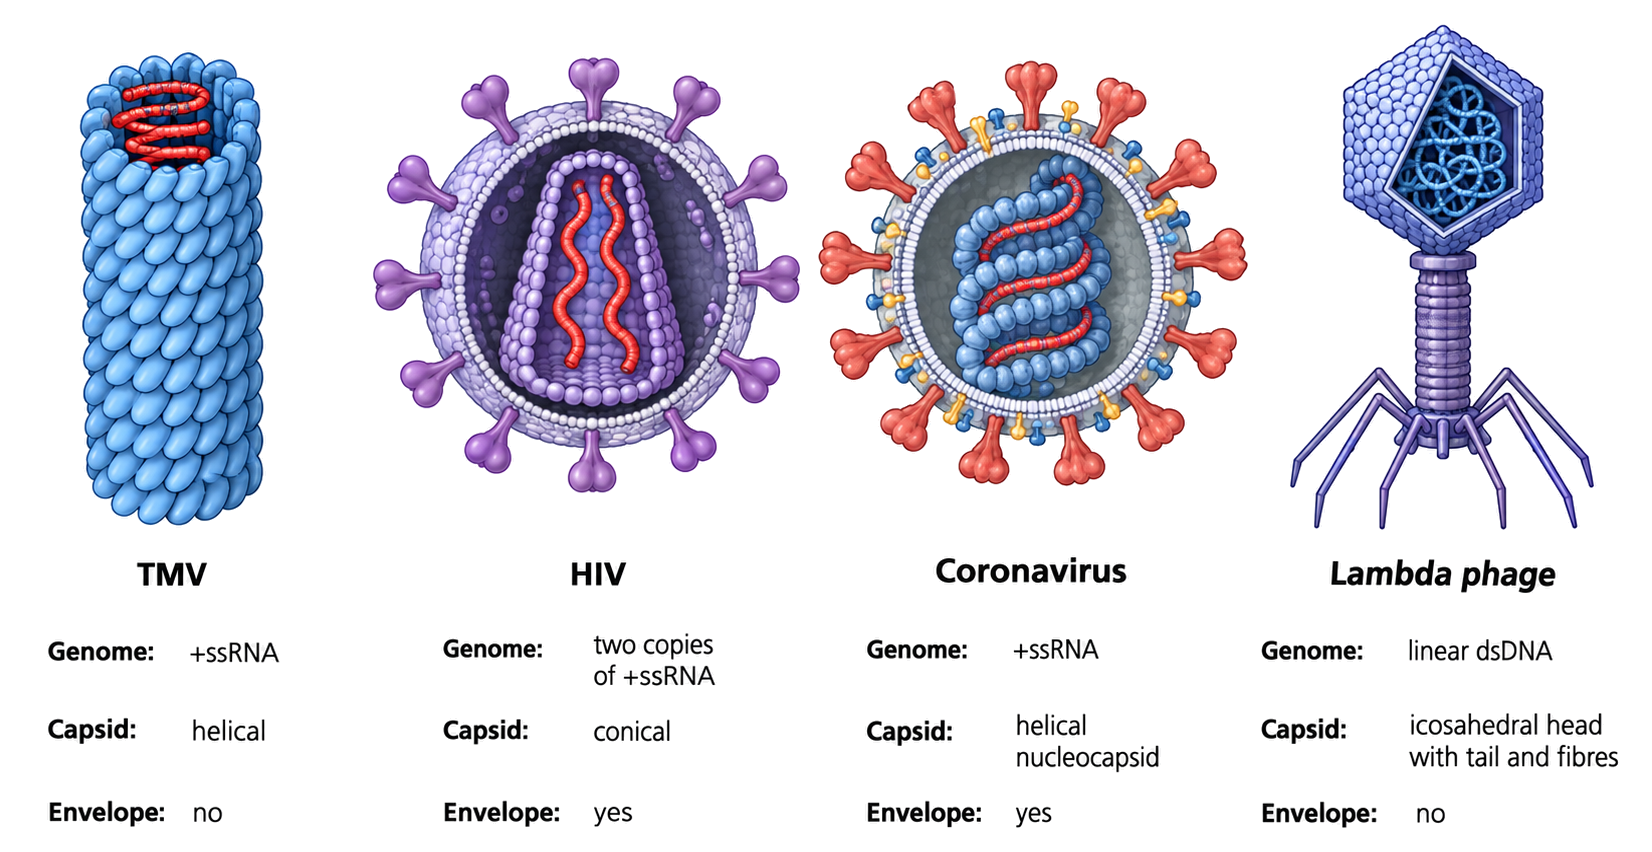
A virus cannot be classified from one feature alone. Its design combines three independent axes: genome form, capsid geometry and envelope status.
Tobacco mosaic virus: single-stranded RNA, helical capsid, no envelope
HIV: two copies of single-stranded RNA, conical capsid, envelope present
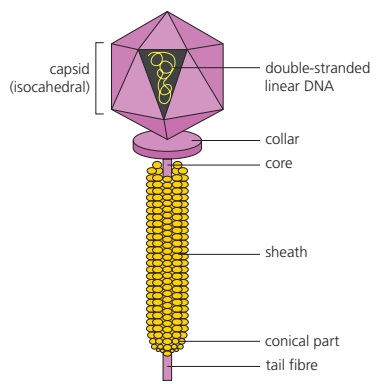
Lambda phage: linear double-stranded DNA, icosahedral head with a complex tail, no envelope
Genome may be DNA or RNA, single- or double-stranded, linear, circular or segmented. Capsids may be helical, polyhedral, conical or complex. An envelope is an additional lipid membrane, not a replacement for the capsid.
Capsid, envelope and glycoproteins solve different problems
HL only
The capsid is assembled from protein subunits and protects the genome. Its geometry also packages the genome efficiently, but a capsid cannot synthesize proteins or supply energy.
In an enveloped virus, host-derived phospholipids surround the capsid. Viral genes encode the surface glycoproteins embedded in that membrane; their shape determines which host-cell receptors the virion can bind.
Receptor binding creates host and tissue specificity and initiates entry. The envelope can aid membrane fusion, but non-enveloped viruses use other entry mechanisms, so an envelope is useful rather than universal.
Lambda phage begins by recognizing and injecting
HL only
Lambda phage infects E. coli because its tail fibres bind specific receptors on the bacterial surface. This molecular match explains why a phage does not infect every bacterial species.
After attachment, the phage injects its linear double-stranded DNA through the cell envelope. The protein capsid remains outside; it is the viral genome inside the bacterium that determines the next route.
If the DNA remains separate and is expressed immediately, infection enters the lytic route. If it integrates into the bacterial chromosome, it begins the lysogenic route.
The lytic route converts one infection into released phages
HL only
1
The tail fibres attach to E. coli, and lambda DNA enters while the capsid remains outside.
2
The viral DNA remains separate from the bacterial chromosome. Host DNA is degraded, freeing nucleotides, while viral genes redirect host enzymes, ribosomes, energy and materials.
3
Lambda DNA is replicated, and viral mRNAs are translated into capsid, tail and lysis proteins.
4
Genome molecules and protein parts self-assemble into complete virions. Assembly must follow synthesis because individual parts are not infectious phages.
5
Viral enzymes weaken the bacterial wall; the cell lyses, dies and releases many phages that can infect neighbouring bacteria.
The lysogenic route copies viral DNA without making virions
HL only
1
After injection, lambda DNA can integrate into the E. coli chromosome. The integrated viral genome is a prophage; the bacterium carrying it is a lysogen.
2
The prophage is copied whenever the host chromosome replicates and is passed to daughter cells during binary fission. No new virions are assembled, so the host is not lysed during this phase.
3
Stress such as DNA damage can trigger induction: the prophage excises from the chromosome, viral genes are expressed, and infection switches into the lytic route.
Genome state separates lytic production from lysogenic inheritance
HL only
Question
Lytic route
Lysogenic route
Where is lambda DNA?
separate from the host chromosome
integrated as a prophage
What is copied?
viral DNA for immediate phage production
host chromosome and prophage together
Are virions made now?
yes
no
What happens to the host?
cell lyses and dies
cell survives and passes the prophage to daughters
What can change the route?
completes with lysis
stress can induce excision and entry into the lytic route
The decisive distinction is not whether viral DNA entered the cell—it does in both routes. The distinction is the state of that DNA after entry, which determines immediate virion production or inherited latency.
Lambda is a temperate phage because the same virus can use either route. Lysogeny postpones virion production; it does not remove the possibility of later lysis.
Viral diversity argues against one universal viral ancestor
HL only
Cellular life shares deeply conserved machinery and genes, supporting common ancestry. Viruses show a different pattern: no gene is shared by every viral group, and their genomes, replication strategies and particle structures are exceptionally diverse.
This pattern supports polyphyly—different viral groups probably arose independently, at different times and by more than one route. It does not identify a separate origin for every virus; it rejects the assumption that one known ancestor explains them all.
All viruses nevertheless share extreme host dependence. That similarity may be convergent evolution: unrelated replicating systems exposed to the same selective problem independently evolved compact transmissible particles that exploit cells.
Three hypotheses describe different routes to viral dependence
HL only
Virus-first: self-replicating molecules existed before or alongside early cells and later became dependent parasites.
Escaped genes (progressive): mobile genetic elements left cells and gained structures for transmission between hosts.
Regressive (reduction): cellular parasites lost genes and cellular structures as host dependence increased.
These are hypotheses, not three stages of one history. Escaped-gene models may fit some small mobile-element-derived viruses, while reduction may fit some large DNA viruses. More than one hypothesis can therefore be correct for different viral lineages.
Rapid viral evolution requires variation and selection
HL only
Mutation creates new alleles during genome replication; recombination or segment reassortment can create new combinations. These processes generate heritable variation before selection acts.
Viruses can evolve rapidly because:
replication enzymes—especially many RNA-dependent polymerases and HIV reverse transcriptase—make frequent uncorrected errors
short generation times expose variants to selection quickly
enormous populations generate many mutations in every infection
repeated transmission exposes variants to changing hosts, immunity and treatments
Selection does not create a needed mutation. A variant already present increases in frequency when it leaves more descendants—for example by replicating faster, transmitting more effectively, evading immunity or surviving an antiviral drug.
High mutation rate alone is not evolution. Population evolution is the change in variant frequencies across generations after mutation, inheritance and differential reproductive success interact.
Antigenic drift and shift change influenza at different scales
HL only
Process
Source of change
Typical result
antigenic drift
accumulated point mutations during replication
gradual alteration of HA or NA antigens within a lineage
antigenic shift
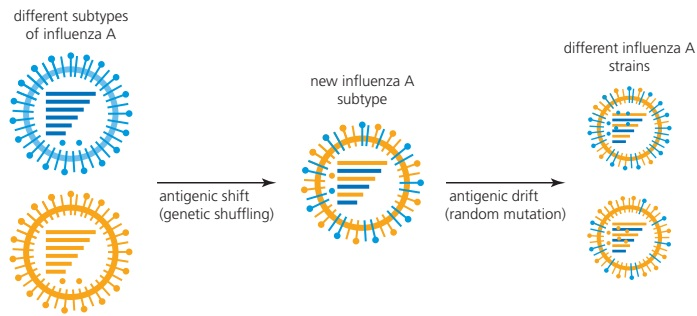
reassortment when different influenza A viruses infect the same cell
abrupt new combination of genome segments and potentially a new subtype
Antibodies bind particular antigen shapes. Drift can gradually reduce recognition and helps explain repeated vaccine updates. Shift can expose a population to a much less familiar antigen combination, so its epidemiological effect may be larger and more sudden.
Shift depends on a segmented genome and co-infection of one host cell; it is not simply a larger point mutation. Drift and shift both generate variation, after which transmission and immunity determine which variants spread.
HIV evolution undermines single-drug treatment
HL only
HIV carries RNA and reverse transcriptase, which copies viral RNA into DNA before that DNA integrates into the host genome. Reverse transcriptase lacks effective proofreading, so copying creates frequent mutations.
Within one person, rapid replication and a large viral population produce many related HIV variants. Most mutations are neutral or harmful, but some alter a protein targeted by an antiviral drug.
A single drug creates strong selection: susceptible variants are suppressed while a resistant variant continues reproducing and becomes more common. The drug selects resistance from existing variation; it does not direct HIV to make the useful mutation.
Combination therapy attacks different viral targets at once. A virion would need several compatible resistance changes to reproduce successfully, greatly reducing the probability that an already resistant variant survives treatment.
Virus synthesis: dependence connects structure, replication and evolution
HL only
Question
Evidence or state to identify
Defensible conclusion
Why must this virus use a host?
genome and capsid but no cytoplasm, ribosomes or independent metabolism
it must redirect compatible cellular machinery
Which lambda route is operating?
viral DNA separate or integrated; virions present or absent
immediate lytic production or lysogenic inheritance
Did all viruses share one origin?
no gene shared by all groups and extreme structural/genomic diversity
several origins are more likely than one universal viral ancestor
Why is a viral population changing?
heritable variants plus different reproductive success
mutation or reassortment supplied variation; selection changed frequencies
The same dependence runs through the chapter: compact viral genomes succeed by using cells. That dependence shapes particle structure and replication, may have evolved by several routes, and creates intense selection whenever host immunity or treatment changes the cellular environment.
Common structural features
HL only
1 mark
Describe one reason that viruses are not considered to be living.
Diversity of virus structure
HL only
7 marks
Describe, with examples, the diversity of structure in viruses.
Lytic cycle
HL only
1 mark
What is a difference between the lytic and the lysogenic cycle of the bacteriophage lambda?
Lysogenic cycle
HL only
3 marks
Explain how the bacteriophage lambda reproduces in the lysogenic cycle.
Rapid evolution in viruses
HL only
2 marks
Outline two reasons for the very rapid rates of evolution in some viruses.